|
Search Term: " ignoring "
The Ultimate Guide to Cellular Longevity: NAD+, Methylation, and Senolytics   
Date:
September 10, 2026 10:57 AM
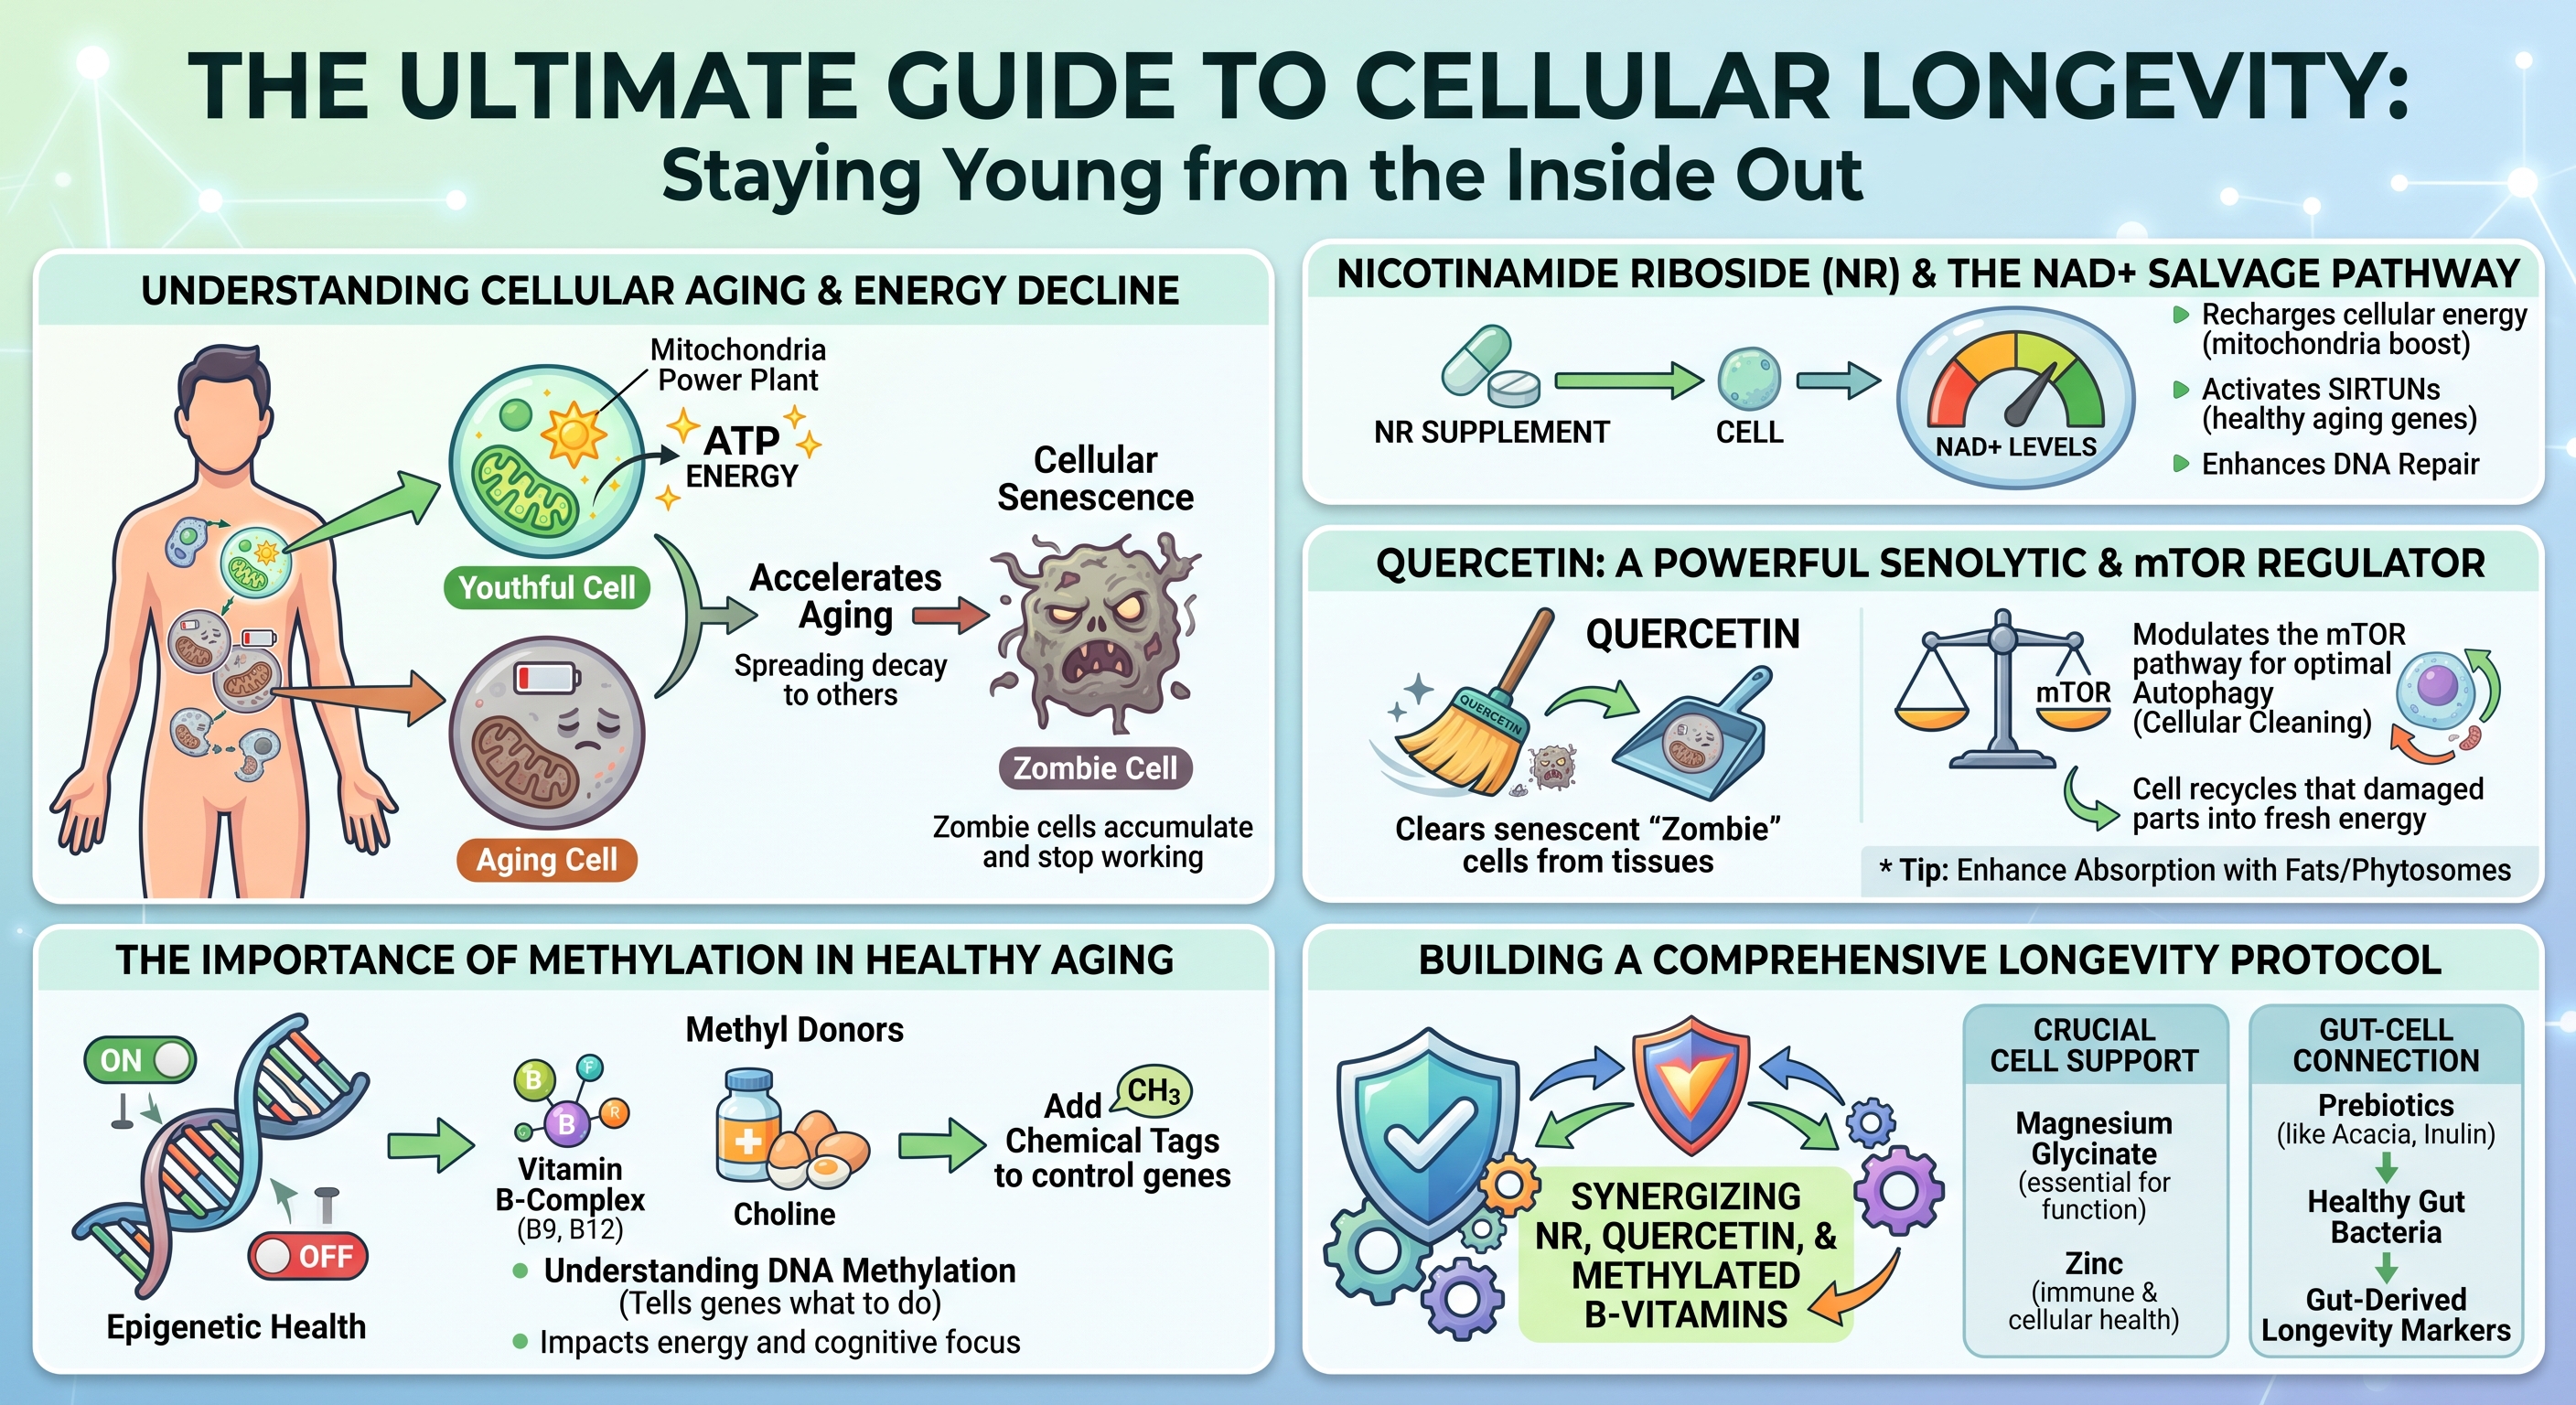
Introduction: Understanding Cellular Aging and Energy DeclineBiological aging represents a progressive decline in cellular maintenance, structural repair, and energy generation. Over decades, tissues experience an attrition of functional reserves, compromised stress resilience, and persistent low-grade systemic inflammation. At the cellular scale, biological degeneration is driven by a failure to generate bioenergetic fuel, repair genetic code, and clear metabolic waste.Cellular aging is characterized by interconnected biological disruptions known as the hallmarks of aging. These encompass genomic instability, epigenetic alterations, mitochondrial decay, loss of proteostasis, and cellular senescence. Rather than operating as isolated occurrences, these phenomena establish a self-reinforcing degenerative cycle: declining cellular power generation impairs enzymatic genetic repair, promoting the accumulation of damaged cells that enter irreversible growth arrest and poison surrounding healthy tissues. Mitigating cellular aging requires examining how microscopic bioenergetic pathways deteriorate and evaluating how targeted nutritional and biochemical interventions can restore cellular homeostasis. The Role of Mitochondria and ATP ProductionEvery biological function - from muscular contraction to continuous DNA replication - depends on adenosine triphosphate (ATP), the primary biochemical energy currency of living systems. Cells produce the vast majority of this energy within mitochondria through oxidative phosphorylation. Within these specialized organelles, metabolic intermediates derived from dietary carbohydrates and lipids donate high-energy electrons to the electron transport chain. The flow of these electrons across protein complexes establishes an electrochemical proton gradient across the inner mitochondrial membrane, driving ATP synthase to manufacture ATP.A youthful cell functions like an efficient municipal power grid, dynamically matching energetic demands with immediate ATP output. However, as biological aging progresses, mitochondrial efficiency declines. The electron transport chain becomes structurally leaky, inadvertently shedding electrons that react with ambient molecular oxygen to produce reactive oxygen species (ROS). While regulated levels of ROS participate in vital intracellular signaling, chronic excess induces widespread oxidative stress. Mitochondria are exceptionally vulnerable to this oxidative burden because they carry their own circular genetic material, known as mitochondrial DNA (mtDNA). Unlike nuclear DNA, mtDNA lacks the protective shielding of histone proteins and possesses rudimentary repair systems. As a result, mtDNA sustains cumulative oxidative damage, encoding increasingly defective electron transport chain proteins. This dynamic generates a bioenergetic deficit: degraded mitochondria synthesize progressively less ATP while emitting greater volumes of damaging free radicals. Deprived of optimal ATP reserves, cells lack the energy necessary to drive vital enzymatic repair cascades, accelerating structural degeneration and functional exhaustion. How Cellular Senescence Accelerates the Aging ProcessWhen healthy cells confront critical physiological damage - such as severe telomere attrition, persistent DNA double-strand breaks, or oxidative stress - they activate protective cell cycle arrest pathways governed primarily by the p53/p21^CIP1 and p16^INK4a/Rb molecular checkpoints. This defensive shutdown, termed cellular senescence, permanently prevents the replication of potentially premalignant or mutated cells.Senescent cells, colloquially known as "zombie cells," enter a state of permanent growth arrest while actively resisting programmed cell death (apoptosis). Over time, these cells accumulate within adipose depots, skeletal muscle, the vascular endothelium, and major organs, largely because immune surveillance and clearance pathways simultaneously lose functional efficiency. The systemic danger of senescent cells stems from their secretome. Rather than remaining biologically inert, senescent cells develop a hyperactive secretory state termed the Senescence-Associated Secretory Phenotype (SASP). The SASP is a destructive mixture of pro-inflammatory cytokines, chemokines, extracellular matrix-degrading matrix metalloproteinases (MMPs), and reactive oxygen species. Through this toxic secretome, even a small burden of senescent cells can impair whole-tissue architecture. SASP factors degrade surrounding structural proteins, induce insulin resistance in neighboring metabolic cells, and biochemically force adjacent healthy cells into secondary senescence. This persistent paracrine signaling fuels chronic, sterile, low-grade systemic inflammation, termed "inflammaging," which accelerates systemic tissue degeneration and elevates susceptibility to degenerative age-related pathologies. Nicotinamide Riboside (NR) and the NAD+ Salvage PathwayThe Biochemistry of NAD+ Depletion Over TimeNicotinamide adenine dinucleotide (NAD+) is an indispensable coenzyme present in every living cell. NAD+ fulfills a dual biological mandate: it serves as a central redox cofactor that shuttles electrons between cellular metabolic reactions, and it functions as an obligatory consumable substrate for regulatory enzymes that preserve cellular viability. In its redox capacity, NAD+ accepts electrons to form NADH during glycolysis, the tricarboxylic acid (TCA) cycle, and fatty acid beta-oxidation, subsequently donating those electrons to Complex I of the respiratory chain to power ATP synthesis.
The primary enzymatic driver of age-related NAD+ destruction is CD38, a membrane-bound glycohydrolase expressed on immune cells that is upregulated in response to chronic SASP exposure. Concurrently, lifelong genotoxic damage causes persistent activation of Poly(ADP-ribose) polymerase 1 (PARP-1), an enzyme that cleaves the glycosidic bonds of NAD+ to assemble branched poly(ADP-ribose) chains at DNA lesion sites. Because PARP-1 consumes NAD+ without directly recycling the molecule, chronic DNA damage depletes intracellular NAD+ pools, impairing bioenergetics and limiting sirtuin activity. How NR Efficiently Boosts Cellular NAD+ LevelsThe mammalian body maintains its NAD+ supply through three distinct biosynthetic routes: the de novo pathway from dietary L-tryptophan, the Preiss-Handler pathway from nicotinic acid (niacin), and the NAD+ Salvage Pathway. The de novo pathway requires substantial energy expenditure, consuming roughly sixty milligrams of dietary tryptophan to yield a single milligram of NAD+. The Preiss-Handler pathway, while effective, can induce cutaneous prostaglandin-mediated flushing at therapeutic intakes. Consequently, the salvage pathway serves as the primary mechanism for maintaining intracellular NAD+ pools.The salvage pathway recycles the breakdown product nicotinamide (NAM), which is released whenever NAD+-consuming enzymes execute their functions. Under normal conditions, cells convert free nicotinamide into nicotinamide mononucleotide (NMN) via the rate-limiting enzyme nicotinamide phosphoribosyltransferase (NAMPT), after which NMN adenylyltransferases (NMNAT1–3) complete the conversion into NAD+. However, NAMPT expression declines with advancing age, chronic inflammation, and metabolic stress, limiting the recycling capacity of the cell. Nicotinamide Riboside (NR) is a naturally occurring pyridine nucleoside that bypasses this enzymatic bottleneck. Upon cellular entry via equilibrative nucleoside transporters, NR is directly phosphorylated into NMN by nicotinamide riboside kinases (NRK1 and NRK2) using a single molecule of ATP. Because the NRK pathway remains intact and robust across the lifespan, NR provides an efficient alternative entry point into the NAD+ salvage cascade. Clinical evaluations in humans confirm the safety, bioavailability, and pharmacokinetics of oral NR supplementation. Randomized, double-blind, placebo-controlled trials reveal that oral NR chloride produces dose-dependent increases in steady-state whole blood NAD+ concentrations. Dosing regimens of 100 mg, 300 mg, and 1,000 mg daily elevate blood NAD+ levels by approximately 22%, 51%, and up to 142%, respectively, within two weeks of administration, maintaining these elevations throughout continuous use. High-resolution metabolomic analyses also demonstrate parallel elevations in nicotinic acid adenine dinucleotide (NAAD), establishing it as a reliable biomarker of active intracellular NAD+ synthesis without hepatic or systemic toxicity. Sirtuin Activation and DNA Repair MechanismsReplenishing intracellular NAD+ supports functions beyond mitochondrial ATP generation. NAD+ functions as an obligatory cofactor for sirtuins (SIRT1 through SIRT7), a family of class III histone and non-histone protein deacetylases that regulate stress resilience, metabolic homeostasis, and cell survival. Sirtuins couple the removal of acetyl groups from target lysine residues to the stoichiometric cleavage of NAD+, producing nicotinamide and O-acetyl-ADP-ribose. In states of NAD+ deficiency, sirtuin enzymes remain inactive regardless of cellular demand.In the nucleus, SIRT1 coordinates defense against cellular decline. When activated by restored NAD+ levels, SIRT1 deacetylates peroxisome proliferator-activated receptor-gamma coactivator 1-alpha (PGC-1a), the master transcriptional coactivator of mitochondrial biogenesis. This deacetylation stimulates mitochondrial replication and assembly, expanding functional respiratory capacity. Concurrently, SIRT1 deacetylates the p65 subunit of nuclear factor-kappa B (NF-kB), suppressing the transcription of pro-inflammatory cytokines. In the mitochondria, SIRT3 utilizes NAD+ to deacetylate metabolic enzymes and superoxide dismutase 2 (SOD2), enhancing the organelle's capacity to neutralize reactive oxygen species. At the same time, cellular NAD+ levels directly regulate genomic integrity through PARP-1. When genotoxic stress or oxidative damage induces single- or double-strand DNA breaks, PARP-1 binds to the damaged termini using its zinc-finger domains. Bound PARP-1 hydrolyzes NAD+ to synthesize extensive, negatively charged poly(ADP-ribose) polymers on itself and adjacent histones. This modification relaxes chromatin architecture and establishes an electrostatic scaffold that recruits base excision repair and homologous recombination complexes. Recent discoveries demonstrate close crosstalk between sirtuins and PARP-1 during DNA repair. PARP-1 recruits SIRT1 to double-strand breaks, where SIRT1 deacetylates the chromatin-remodeling ATPase BRG1 to displace nucleosomes and facilitate homologous recombination. However, because PARP-1 and SIRT1 draw from the same intracellular NAD+ pool, severe NAD+ depletion forces a biological compromise: PARP-1 consumes the scarce remaining cofactor to address DNA damage, leaving sirtuins deactivated. Restoring NAD+ via NR prevents this deficit, enabling concurrent genomic repair and sirtuin-mediated metabolic defense. Quercetin: A Powerful Senolytic and mTOR RegulatorClearing Senescent "Zombie" Cells from TissuesThe accumulation of senescent cells has driven interest in senolytics: molecules that selectively eliminate senescent cells while sparing healthy, non-senescent populations. Senolytic agents exploit a specific vulnerability in senescent cells. Because senescent cells produce cytotoxic, pro-inflammatory SASP factors that would normally induce their own death, they become dependent on upregulated Senescent Cell Anti-Apoptotic Pathways (SCAPs) to survive. The SCAP network involves anti-apoptotic proteins (such as BCL-2 and BCL-xL), the PI3K/Akt kinase cascade, and cyclin-dependent kinase inhibitors.Quercetin is a polyphenolic flavonoid found in capers, red onions, apples, and the flower buds of Sophora japonica. Beyond its classical antioxidant properties, quercetin functions as a senolytic compound that exerts multi-target inhibitory effects across the SCAP network. By inhibiting the upstream PI3K/Akt survival axis and downregulating anti-apoptotic defenses, quercetin disrupts the signaling that protects senescent cells from intrinsic apoptosis. Deprived of these survival signals, senescent cells undergo programmed cell death. Preclinical studies demonstrate that senolytic protocols utilizing quercetin - often combined with the tyrosine kinase inhibitor dasatinib - reduce senescent cell burden across multiple tissues. This targeted clearance lowers circulating SASP factors, attenuates tissue fibrosis, restores endothelial reactivity, and improves functional health span. By removing senescent cells, quercetin mitigates the primary driver of chronic, low-grade inflammaging. Modulating the mTOR Pathway for Optimal AutophagyThe mechanistic Target of Rapamycin (mTOR) is an evolutionarily conserved serine/threonine protein kinase that coordinates cellular metabolism by balancing anabolic growth with catabolic recycling. Operating within two multiprotein complexes - mTORC1 and mTORC2 - the mTOR pathway integrates signals from amino acids, growth factors, and intracellular energy levels. In nutrient-rich environments, mTORC1 promotes protein synthesis, lipogenesis, and cellular growth, while suppressing catabolic breakdown. Conversely, nutrient scarcity downregulates mTORC1, activating autophagy.Autophagy is an intracellular degradation system that packages damaged organelles, misfolded protein aggregates, and biological debris into double-membraned autophagosomes for lysosomal degradation and recycling. A specialized branch of this pathway, mitophagy, selectively targets and clears damaged mitochondria. In modern metabolic conditions characterized by continuous caloric intake, mTORC1 can remain persistently active. This persistent signaling suppresses autophagy, causing damaged organelles and toxic aggregates to accumulate within tissues. Quercetin functions as a natural modulator of mTOR signaling. By inhibiting upstream PI3K/Akt signaling and activating intracellular energy sensors, quercetin attenuates overactive mTORC1, mimicking the metabolic effects of caloric restriction. This down-regulation relieves inhibition on the ULK1 autophagy initiation complex, stimulating both general autophagy and mitophagy. As autophagy proceeds, cells clear protein aggregates and eliminate damaged mitochondria, supporting cellular longevity and proteostasis. Enhancing Absorption: Phytosomes and Dietary FatsDespite the biological activities of quercetin identified in experimental models, its clinical translation has historically been limited by poor oral bioavailability. Raw quercetin aglycone is a crystalline, hydrophobic polyphenol with poor solubility in water and gastrointestinal fluids. When ingested in unformulated powder forms, quercetin molecules aggregate in the gut lumen, resisting dissolution and passive absorption. Consequently, the vast majority of an unformulated dose passes into the colon unabsorbed, where it undergoes microbial degradation without reaching meaningful systemic concentrations.To address these pharmacokinetic limitations, advanced delivery systems such as phytosomes were engineered. A phytosome is a 100% food-grade molecular complex where individual polyphenolic molecules are bound to dietary phospholipids, typically sunflower-derived phosphatidylcholine. Unlike a classical liposome - which encapsulates water-soluble compounds inside an aqueous core enclosed by a lipid bilayer - a phytosome forms an amphiphilic complex at the molecular level. The polar head of the phosphatidylcholine molecule forms hydrogen bonds with the hydroxyl groups of the quercetin molecule, while its lipophilic fatty acid tails extend outward. This structural arrangement shields the polar regions of the flavonoid, creating a lipid-compatible complex that integrates smoothly into the intestinal mucosa.
The Importance of Methylation in Healthy AgingVitamin B-Complex and Choline as Essential Methyl DonorsMethylation is an essential biochemical process occurring billions of times each second across all human tissues. It involves the transfer of a single-carbon unit - a methyl group consisting of one carbon atom bound to three hydrogen atoms - (CH3) - from a donor molecule to diverse recipients, including DNA, RNA, structural proteins, neurotransmitters, and membrane phospholipids. This transfer of one-carbon units is coordinated by the methionine-homocysteine cycle, which sustains genetic stability, detoxification pathways, and cellular repair.At the center of this pathway sits S-adenosylmethionine (SAM), the universal methyl donor in human biology. When a methyltransferase enzyme transfers a methyl group from SAM to an acceptor molecule, SAM is converted into S-adenosylhomocysteine (SAH). SAH functions as a potent competitive inhibitor of intracellular methyltransferases. To maintain functional methylation, SAH is rapidly hydrolyzed into homocysteine, a sulfur-containing amino acid that must be remethylated or cleared through transsulfuration. Homocysteine clearance proceeds through two distinct remethylation pathways. The primary route operates across most tissues via the enzyme methionine synthase, which requires vitamin B12 in its active methylcobalamin form. Methionine synthase transfers a methyl group from 5-methyltetrahydrofolate (5-MTHF, the active form of folate) to homocysteine, regenerating methionine. The ongoing production of 5-MTHF depends on the enzyme methylenetetrahydrofolate reductase (MTHFR), which utilizes riboflavin (vitamin B2) as a cofactor. Alternatively, excess homocysteine can be routed into the transsulfuration pathway by vitamin B6 (as pyridoxal-5'-phosphate) to synthesize cystathionine, cysteine, and ultimately the antioxidant glutathione. A secondary remethylation pathway, active predominantly in hepatic and renal tissues, bypasses folate entirely. In this route, dietary choline is oxidized to betaine (trimethylglycine or TMG). The enzyme betaine-homocysteine S-methyltransferase (BHMT) then transfers a methyl group from betaine directly to homocysteine, yielding methionine and dimethylglycine. When dietary intake of active B-vitamins or choline is insufficient, or when genetic variations like MTHFR polymorphisms reduce pathway flux, the methylation cycle slows. Homocysteine accumulates in circulation, promoting vascular and neurological inflammation, while SAM reserves decline, restricting cellular methylation capacity. Understanding DNA Methylation and Epigenetic HealthEvery somatic cell in an organism carries an identical genetic code. Cellular differentiation and tissue-specific functions are governed by the epigenome: a regulatory layer of chemical modifications that dictates gene expression without altering underlying DNA sequences. DNA methylation represents the primary and most stable epigenetic modification. In this process, DNA methyltransferase (DNMT) enzymes utilize methyl groups donated by SAM to add a methyl tag to cytosine bases adjacent to guanine residues, forming 5-methylcytosine within CpG dinucleotide sites.Under physiological conditions, DNA methylation maintains genomic stability and coordinates transcription. Methylation of promoter regions condenses chromatin, repressing transposable elements and silencing genes inappropriate for a given cell type. Conversely, hypomethylated promoters maintain an open chromatin state, allowing transcription factors to bind and initiate gene expression. During biological aging, this epigenetic landscape undergoes progressive dysregulation, a phenomenon termed "epigenetic drift". Aging cells experience global hypomethylation alongside focal hypermethylation of specific gene promoters. Global loss of methyl tags destabilizes the genome, activating retrotransposons and pro-inflammatory pathways. Simultaneously, hypermethylation at targeted promoter sites silences critical tumor suppressor genes and DNA repair complexes. This systematic change in DNA methylation patterns is consistent across populations, allowing researchers to develop molecular "epigenetic clocks". Algorithms such as the Horvath clock, PhenoAge, and GrimAge quantify biological age by profiling the methylation status of specific CpG sites across the genome. These clocks assess whether individuals are aging faster or slower than their chronological years. Ensuring a steady supply of methyl donors and preventing unnecessary SAM depletion supports DNMT activity, maintaining epigenetic patterns and genomic stability. How the Methylation Cycle Impacts Energy and Cognitive FocusBeyond long-term epigenetic regulation, the methylation cycle directly modulates immediate biochemical processes that govern daily energy, neurotransmission, and cognitive focus. Compromised methylation capacity frequently manifests as cognitive slowing, executive fatigue, and reduced physical stamina.A major consumer of methyl reserves is the endogenous synthesis of creatine. Approximately 40% of all SAM-derived methyl groups in the human body are utilized by guanidinoacetate N-methyltransferase (GAMT) in the liver to synthesize creatine. Creatine then translocates to the brain and skeletal muscle, where it is phosphorylated into phosphocreatine. Phosphocreatine functions as a rapid energy buffer, donating a high-energy phosphate group to regenerate ADP into ATP in milliseconds during demanding physical or cognitive tasks. When methyl donor availability falls, endogenous creatine synthesis drops, depleting phosphocreatine reserves and increasing susceptibility to neuromuscular and cognitive fatigue. Methylation is equally central to central nervous system architecture. SAM provides methyl groups to convert phosphatidylethanolamine into phosphatidylcholine, the predominant phospholipid comprising neuronal cell membranes and the myelin sheaths that insulate axons. Intact myelin preserves rapid action potential conduction throughout the nervous system. Furthermore, free choline derived from this pathway is the direct precursor to acetylcholine, the neurotransmitter required for attention, working memory, and learning. The methylation cycle also governs monoamine neurotransmitter metabolism. SAM is required for the synthesis of adrenaline (epinephrine) from noradrenaline, while catechol-O-methyltransferase (COMT) relies on SAM to degrade dopamine and norepinephrine within the prefrontal cortex. Sluggish methylation disrupts this balance, contributing to cognitive fatigue, mood variability, and impaired mental performance. Building a Comprehensive Longevity ProtocolSynergizing NR, Quercetin, and Methylated B-VitaminsLongevity supplementation often falters when single molecules are administered in isolation, ignoring interconnected metabolic pathways. Designing an effective cellular longevity protocol requires combining complementary mechanisms that reinforce one another while preventing secondary metabolic deficits. The combination of Nicotinamide Riboside, Quercetin Phytosome, and Methylated B-Vitamins illustrates this multi-target synergy.This synergy is grounded in the direct biochemical intersection between the NAD+ salvage pathway and the methylation cycle. When high-dose NR is supplemented to boost systemic NAD+, sirtuins and PARP enzymes consume the newly synthesized cofactor, generating substantial quantities of free nicotinamide (NAM). This intracellular nicotinamide faces two primary metabolic fates: it can be recycled back into NAD+ through the NAMPT-dependent salvage loop, or it can be cleared via methylation. When the influx of nicotinamide exceeds salvage recycling capacity, the excess is cleared to avoid feedback inhibition of sirtuin enzymes. To accomplish this, the enzyme nicotinamide N-methyltransferase (NNMT) transfers a methyl group from SAM directly onto nicotinamide, forming 1-methylnicotinamide (1-MNA/MNAM), which is subsequently excreted in urine. Prolonged, high-dose precursor administration without nutritional methyl support can elevate NNMT flux, depleting intracellular SAM reserves. As methyl groups are consumed clearing nicotinamide, the cellular SAM-to-SAH ratio falls, which can elevate circulating homocysteine and reduce methyl availability for DNA methylation and neurotransmitter synthesis. Co-administering a fully methylated B-complex alongside choline or betaine addresses this potential bottleneck. Providing active methyl donors (such as 5-MTHF, methylcobalamin, and betaine) maintains the one-carbon donor pool. Even during increased NNMT activity, SAM pools remain stable, protecting DNA methylation fidelity and maintaining homocysteine within safe parameters. Quercetin reinforces this protocol through complementary mechanisms. By clearing senescent cells and reducing SASP-mediated inflammation, quercetin downregulates CD38, the primary enzyme responsible for age-related NAD+ degradation. Suppressing CD38 prevents unnecessary breakdown of newly synthesized NAD+, enhancing the efficiency of NR supplementation. Furthermore, while NR provides the NAD+ necessary to activate SIRT1-driven mitochondrial biogenesis, quercetin concurrently modulates mTORC1 to stimulate autophagy. This coordinated action ensures that newly generated mitochondria operate in an environment cleared of proteotoxic cellular debris. The Crucial Role of Magnesium Glycinate and Zinc in Cellular FunctionLongevity protocols require essential mineral cofactors to function efficiently. Without adequate divalent minerals acting as enzymatic cofactors and structural stabilizers, metabolic longevity pathways cannot operate at full capacity. Among these, magnesium and zinc are required for cellular repair, genomic stability, and energy production.Magnesium serves as an obligatory cofactor in over 300 enzymatic reactions, primarily through its interaction with ATP. In biological systems, ATP exists predominantly as a chelate with a divalent magnesium ion, forming biologically active Mg2+ -ATP. Every enzymatic reaction that synthesizes, transfers, or consumes cellular energy - including the enzymes of the NAD+ salvage pathway (NRK and NMNAT) and DNA polymerases - strictly requires Mg2+ -ATP as its substrate. Magnesium deficiency impairs these phosphorylation reactions, reducing the cellular utilization of NAD+ precursors. Additionally, magnesium is an essential cofactor for the enzymes that activate dietary B-vitamins into their active forms. Supplying magnesium as magnesium glycinate provides high gastrointestinal bioavailability, minimal laxative effect, and yields glycine to support inhibitory neurotransmission and restful sleep. Zinc serves as a vital structural component for more than 3,000 human transcription factors and enzymatic proteins. Its most prominent structural role in longevity occurs within zinc-finger motifs. These are specialized protein conformations stabilized by a zinc ion coordinated to cysteine and histidine residues. The DNA damage sensor PARP-1 utilizes three zinc-finger domains to identify, track, and physically bind to single- and double-strand DNA breaks. Without adequate intracellular zinc, PARP-1 cannot properly assemble or dock onto damaged chromosomes, impairing DNA repair and increasing genomic instability. Zinc is also an obligatory structural component of copper/zinc superoxide dismutase (Cu/Zn-SOD or SOD1), the primary cytosolic antioxidant enzyme that dismutates superoxide radicals into hydrogen peroxide, protecting mitochondrial membranes and nuclear DNA from premature senescence. Integrating Prebiotics (like Acacia and Inulin) for Gut-Derived Longevity MarkersA comprehensive cellular longevity framework must extend beyond somatic tissues to encompass the gut microbiome. The intestinal microbiome functions as a central regulator of systemic inflammatory tone, immune development, and metabolic signaling. Age-associated dysbiosis - characterized by the loss of beneficial commensals and an overgrowth of pathobionts - frequently leads to breakdown of the intestinal barrier.The gut epithelium consists of a single-cell monolayer sealed by tight junction proteins, including zonula occludens-1 (ZO-1), occludin, and claudins. When this physical barrier is disrupted by poor dietary fiber intake or dysbiosis, gut permeability increases. This allows lipopolysaccharide (LPS), a component of the outer membrane of Gram-negative bacteria, to enter the portal and systemic circulation. The resulting "metabolic endotoxemia" activates Toll-like receptor 4 (TLR4) on immune cells, inducing NF-kB and systemic pro-inflammatory cytokine production. This persistent gut-derived inflammation exacerbates the SASP, accelerates tissue senescence, upregulates CD38, and drains systemic NAD+ reserves.
These short-chain fatty acids, particularly butyrate, exert direct protective effects on systemic longevity. Butyrate provides the primary metabolic fuel for colonic epithelial cells, supplying more than 70% of their baseline energy needs and supporting mitochondrial function within colonocytes. Furthermore, SCFAs upregulate the expression of epithelial tight junction proteins (ZO-1, occludin, and claudin-1), restoring intestinal barrier integrity and preventing the translocation of inflammatory LPS into systemic circulation. Systemically absorbed butyrate also functions as an endogenous histone deacetylase (HDAC) inhibitor, suppressing pro-inflammatory gene expression and supporting regulatory T cell (T_reg) development. Reducing metabolic endotoxemia dampens systemic inflammation, protecting vascular function and preventing premature NAD+ depletion. Conclusion: The Integrated Cellular Longevity MatrixCellular longevity is achieved not by addressing isolated biomarkers in isolation, but by systematically supporting interconnected biological pathways. As bioenergetic capacity declines, cellular senescence accelerates, epigenetic patterns degrade, and gut barrier integrity weakens. A comprehensive approach addresses these biological vulnerabilities simultaneously.
Quercetin Phytosome clears senescent cells and modulates mTORC1, stimulating autophagy while dampening the inflammatory SASP cascade that accelerates CD38-mediated NAD+ destruction. Methylated B-vitamins, active folate, and choline replenish SAM reserves, balancing the methyl requirements of NNMT-mediated nicotinamide clearance, preserving epigenetic DNA methylation, and maintaining neurotransmitter production. Magnesium glycinate and zinc provide the structural and catalytic foundation required for ATP utilization, B-vitamin activation, and PARP-1 zinc-finger DNA repair docking. Finally, prebiotic fibers generate short-chain fatty acids like butyrate, reinforcing the intestinal barrier and preventing metabolic endotoxemia from fueling systemic inflammation. By coordinating energy replenishment, cellular waste clearance, epigenetic maintenance, and the suppression of systemic inflammation, this unified approach directly addresses the underlying drivers of cellular aging to support long-term physiological vitality.
--
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=6650) What's The Difference Between Pre & Probiotics? 
Date:
May 09, 2017 11:44 AM
Maintaining good digestive health is paramount to overall good health and physical well-being. Much of digestive health is predicated on the balance of bacteria in the digestive system, because it dictates how well nutrients are absorbed as well as the ability to fight infection. Ignoring issues associated with digestive health may lead to problems such as inflammatory bowel disease, diabetes, and other issues that can have a dramatic influence on the overall health of a person. Key Takeaways:
"Research is showing that our gut flora performs pivotal roles in metabolism, nutrient digestion, absorption and synthesis, as well as immune function, hormonal regulation and disease prevention." Read more: https://www.thehealthychef.com/2017/05/whats-the-difference-between-pre-probiotics/
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=4573) WikiLeaks emails mention aspartame, acknowledging it puts holes in mice brains
Date:
November 23, 2016 10:59 AM
Aspartame is bad for us and has been for some time. There are many negative effects of aspartame recorded over the last 20 plus years. People still have done nothing to get rid of this horrible thing because it makes things appear to be better for you. People are just ignoring scientific evidience. Key Takeaways:
"Unfortunately, the history of how aspartame came to be a societal mainstay is not a sweet one." Reference: //www.naturalnews.com/055991_WikiLeaks_aspartame_chemical_sweeteners.html
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=3494) These are the biggest mistakes people make when trying to eat healthy
Date:
November 15, 2016 07:04 AM
There are some common pitfalls to avoid when you decide to start eating healthier. Just because something is labeled “healthy” doesn’t make it so. Check your labels and know your ingredients and then be sure to keep your portions under control as well. You still need to count your calories when you are eating healthy so you know if you are eating too much or too little, as both are common problems. Key Takeaways:
"ignoring moderation because "it's healthy!" - so you're eating fresh, whole foods." Reference:
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=3446) Fennel
Date:
June 30, 2008 04:47 PM
If there has ever been an overlooked vegetable, it would definitely be fennel. Some people have an aversion to its licorice-like scent, while others feel as if fennel is a bizarre and obscure vegetable that they have no interest in learning how to prepare. However, those who have discovered it know that ignoring fennel is a waste of a versatile vegetable’s amazing flavor and healthful benefits. Even those who already cook with fennel might find that they aren’t taking advantage of its versatility. For example, many people use only the delicate, lacy parts of fennel as a flavor-enhancing garnish for soups or salads. Others stick to just using the green-white bulbs, while tossing the remaining pieces aside. However, there’s no season like now to start using and enjoying all the parts of fennel. Fennel is available from autumn until early spring and both its stems and bulbs have been found to contain many nutrients. Fennel spice, which is made from the vegetable’s seeds, can be found year round, as it is one of five spices in Chinese five-spice powder. One cup of raw, sliced fennel is a huge source of vitamin C, folic acid, fiber, and potassium. History has shown that fennel can be taken to alleviate bad breath, indigestion, intestinal spasms, cramps, and gas. It is thought that Puritans chewed the seeds in order to tame hunger during fasts. Recently, scientists have found that fennel contains antioxidants which promote good health. In order to gain these healthful benefits, be sure to purchase white or pale-green fennel that has clean, firm bulbs. The bulbs should not be split, bruised, or spotted, while the stalks that grow from the bulb should be relatively straight. Additionally, the vegetable’s fronds would be green but not flowering because blooms indicate that the bulb is past maturity. When consumed right away, fennel is at its best. But, it can be kept in the crisper for up to four days. Be sure to wash it before using its base in hors d’oeuvres, salads, and gratins. Also, make sure to reserve its fronds in order to enhance dishes in a potent way. With such versatility in the kitchen, there is absolutely no excuse not to include fennel in your meals this season. Once you discover that fennel is both crunchy and slightly sweet, you will want to incorporate it into many of your daily meals. Thankfully, fennel can enhance many dishes and make them extraordinary. Here are some quick ideas for using fennel this season. You can thinly shave the desired amount of a fennel bulb and toss it with a bit of olive oil, fresh lemon juice, and a small amount of Parmesan cheese to make a fennel salad at moment’s notice. Another option is sauté sliced fennel with equal parts of onion and bell pepper in order to make a simple vegetarian side dish. One can take advantage of fennel’s ability to enhance flavors by adding fennel with tuna or grilled sea bass. Fennel can also be cut vertically, leaving bulb, stalk, and leaves intact and then brushed with olive oil and grilled until lightly browned. Another idea is to garnish your favorite vegetable soup with coarsely chopped fennel fronds.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=1829) Adapt To The Stresses Of Life with Herbal Adaptogens
Date:
October 18, 2007 11:13 AM
Life today places a number of different types of stresses upon us. There are the normal stresses of living, of facing problems at work, financial worries and family stresses. Schedules are becoming busier as we try to pack more and more into each day, and relaxation time is cut to a minimum. For many of us, the stress starts when we waken and rush through breakfast, if we have time for one, to catch the bus or train to work, or to slip into the morning traffic rush that takes us an hour to travel 10 miles or less. Once at work we have problems to deal with that continue throughout a rushed lunch period, and then back to the stress of trying to return home in the evening to open the bills and check if we have enough in the bank to pay them. However, that is not all. Our environment is continually changing, and our bodies are subject to the stresses of pollution from the planes, trains and automobiles, not to mention the pesticides, preservatives plastics and harsh lighting. The noise of air conditioning and the continual musak of the stores and shopping malls and everything else that goes to completely stress us out, weekdays and weekends. That is ignoring the smog, the disappearing ozone layer and increased UV radiation, the greenhouse effect and global warming, El Nino and everything else that causes worry or affects the delicate balance of the body’s biochemistry. Rather than adapting to our environment we are continually striving to adapt the environment to suit our needs. We should develop a flexibility of mind and body so that we can survive these modern-day stresses, and this is where the substances known as adaptogens are important. Adaptogens help us to adapt to the environment and withstand the stresses of modern life. The term was first used by Russian N.V. Lazarev in 1947 who defined an adaptogen as a substance meeting three specific criteria: it should cause a minimal disruption to the normal physiological function of the body, it must work by means of a range of chemical, physical and biochemical factors rather than through one specific action and must have an overall effect of normalization, so that no condition is aggravated to improve another. There are a large number of identified adaptogens, among them several forms of ginseng: Panax, American, Siberian and Japanese; licorice, schizandra berries, rhodiola and others. These adaptogens tend to work in the body by improving the body’s availability and use of energy, improving the efficiency of removal of the metabolic waste and by-products, supporting the adrenal function so that the effects of stress are reduced or countered, improving the utilization of oxygen and helping to build up body tissue. In general the body works more efficiently in generating and using energy, muscle tissue and counteracting the effects of modern day stress, both environmental and psychological. Of the ginsengs, Panax is very expensive for regular use, although many people prefer it. However, studies have shown that Siberian, or eleuthero ginseng, is a stronger adaptogen that Panax which is also called Korean or Chinese ginseng. In fact the other forms, including American and Japanese, tend to over-stimulate the body, and can also cause unwanted side effects such as constipation and over-excitement. The Siberian ginseng tends not to show these symptoms. Siberian ginseng contains seven active substances known as eleutherosides A – F which are not present in the other ginsengs. These substances appear to have several properties that have been clinically proven. For example, they relieve insomnia, one of the symptoms of stress, high and low blood pressure, bronchitis, various forms of neuroses and, it is claimed, also some types of cancer. Siberian ginseng also allows humans to withstand noise, heat and extra stresses caused by severe workloads. It improves athletic performance and allows people to improve their work output under a variety of stresses. Athletes can train harder and recover quicker. Another adaptogen is schizandra berries (also called schizandra chinensis and magnolia vine). Chinese herbalists class medicinal herbs by the five different flavors, sour, bitter, salty, acrid and sweet. Schizandra berries possess all five, and are therefore considered by the Chinese to balance all the systems of the body. It is used in the West as a stress reducing adaptogen and is also included in sports and weight loss formulae. It helps insomnia and improves endurance and mental coordination. Schizandra is believed to be a good tonic for the liver and is often used in combination with Siberian ginseng (eleuthero) and licorice. The latter is another popular herb in China that is said to be a good tonic for the spleen. Licorice itself is a known anti-inflammatory since it contains flavanoids and saponins that promote the immune system. Licorice is thought be a useful supplement for HIV patients due to its effect on the immune system. It also increases corticosteroid levels by inhibiting the liver’s ability to break down adrenal hormone. However, people with high blood pressure should be careful with licorice since it can cause sodium retention. Like any other medication, you should seek your physician’s advice if you have any existing conditions. Rhodiola, also referred as roseroot, is used for improved memory and enhanced vitality and it can also be used as a mood modifier. It is used by athletes of all types for increased strength and endurance, and improved cardiovascular and muscle recovery time. The Russians call it ‘Golden Root’ and it is a safe and effective adaptogen. More and more people are turning to adaptogens to help them cope with the hustle and bustle of their daily lives, and they are becoming increasingly available from ordinary health stores. If you are finding it difficult to stay energetic and active then try them out. Not all work with every individual, but there is a large variety to choose from and most people are able to find an adaptogen that suits them and enables them to adapt to the stresses of daily life.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=1596) Lowering cholesterol safely 
Date:
July 27, 2005 04:10 PM
Lowering cholesterol safely. By Kim Vanderlinden, N.D., D.T.C.M. Atherosclerosis and its complications are major causes of death in the United States and have reached epidemic proportions throughout all of the Western world. Heart disease accounts for 36% of all deaths among Americans and ranks as the number-one killer; stroke; another complication of atherosclerosis; is the third most common cause of death. Foremost in the prevention and treatment of heart disease is the reduction of blood cholesterol levels. The evidence overwhelmingly demonstrates that elevated cholesterol levels greatly increase the risk of death due to heart disease. The first step in reducing risk for heart disease is keeping your total blood cholesterol level below 200 mg/dl (milligrams per deciliter). Not all cholesterol is bad; it serves many functions in the body, including the manufacture of sex hormones and bile acids. Without cholesterol, many body processed would not function properly. Cholesterol is transported in the blood by molecules known as lipoproteins. Cholesterol bound to low density lipoprotein, or LDL, is often referred to as the “bad” cholesterol, while cholesterol bound to high-density lipoprotein, or HDL, is referred to as the “good” cholesterol. LDL cholesterol increases the risk of heart disease, strokes, and high blood pressure, while HDL cholesterol actually protects against heart disease. LDL transports cholesterol to the tissues. HDL, on the other hand, transports cholesterol to the liver for metabolism and excretion from the body. Therefore, the HDL-to-LDL ratio largely determines whether cholesterol is being deposited into tissues or broken down and excreted. The risk for heart disease can be reduced dramatically by lowering LDL cholesterol while simultaneously raising HDL cholesterol levels. Research has shown that for every one percent increase in HDL levels, the risk for a heart attack drops three to four percent. Dietary cholesterol Dietary cholesterol is a major risk factor in developing atherosclerosis. The evidence is substantial. However, several studies have shown that a lower dietary cholesterol intake was associated with up to a 37% lower risk of death from any cause, or an increased life expectancy of roughly 3.4 years. Although dietary cholesterol intake is an important contributor to atherosclerosis, most of the cholesterol in the body is actually manufactured in the liver. Reducing dietary cholesterol alone is not always sufficient to lower blood cholesterol levels. Common drugs In an attempt to reduce blood cholesterol levels, many physicians are ignoring the need to give dietary recommendations and are instead utilizing drugs as the primary treatment. Using drugs before diet is clearly not the best approach, in terms of both effectiveness and cost. In fact, the Report of the National Cholesterol Education Program Expert Panel on Detection, Evaluation, and Treatment of High Cholesterol in Adults clearly states: “Dietary therapy is the primary cholesterol-lowering treatment.” The drugs lovastatin (Mevacor), prevastin (Pravachol), and simvastatin (Zocor) are commonly used to lower blood cholesterol levels. The main side effect of these drugs is liver damage. In fact, due to the seriousness of the possible adverse effects on the liver, it is necessary to have periodic blood tests to determine if the drug is harming the liver. Other side effects include: muscle breakdown, muscle pain, nausea, diarrhea, flatus, abdominal pain, headache, and skin rash. The most important first approach to lowering a high cholesterol level is to follow a healthful diet and lifestyle. The dietary changes are simple: Eat less saturated fat and cholesterol by reducing or eliminating the amounts of animal products in the diet; increase consumption of fiber-rich plant foods (fruits, grains, and legumes); and lose weight, if necessary. Lifestyle changes include; Regular aerobic exercise; stop smoking; and reduce or eliminate consumption of coffee (both caffeinated and decaffeinated). Here are the six key recommendations of U.S. Surgeon General, American Heart Association, and the National Research Council’s Committee on Diet and Health:
Natural alternatives When there is a need for additional support to the dietary and lifestyle practices that can lower cholesterol levels, it simply makes more sense to use safer and more effective natural alternatives. When evaluating overall effectiveness, both LDL and HDL cholesterol levels must be taken into consideration. When you look at the cost, safety, and effectiveness, it is clear that natural alternatives are substantially superior to standard drug therapy. Keep in mind that the natural alternatives discussed are, just like the dugs, still best utilized in a comprehensive program that stresses a healthful diet and lifestyle. Niacin, or vitamin B3, has long been used to lower cholesterol levels. In fact, niacin is recommended by the National CholesterolEducation Program as the first “drug” to use to lower blood cholesterol levels. The safest form of niacin at present is known as inositol hexaniacinate. This form of niacin has long been used in Europe to lower cholesterol levels and also to improve blood flow. It yields slightly better results than standard niacin, but is much better tolerated, both in terms of flushing and, more importantm long term side effects. Gugulipid is the standardized extract of the mukul myrrh tree that is native to India. Several clinical studies have confirmed that gugulipid has an ability to lower both cholesterol and triglyceride levels. Typically, cholesterol levels will drop 14% to 27% in a four- to twelve-week period, while triglyceride levels will drop from 22% to 30%. The dosage of gugulipid is based on its guggulsterone content. Clinical studies have demonstrated that gugulipid extracts standardized to contain 25 mg of guggulsterone per tablet given three times per day is an effective treatment for elevated cholesterol levels, elevated triglyceride levels, or both. Garlic and onions exert numerous beneficial effects on the cardiovascular system, including lowering blood lipids and blood pressure. Numerous studies have demonstrated that both garlic and onions are effective in lowering LDL-cholesterol and triglycerides while simultaneously raising HDL-cholesterol levels. Final Comments Without question, the best approach to lowering cholesterol levels is through diet and lifestyle modifications. When additional support is require, there are safer and more effective natural alternatives to commonly prescribed drugs. The goal of therapy, whether natural or synthetic, is to get blood lipid levels down into target ranges as quickly as possible. Once the target range has been achieved, begin reducing the amount of medicine by half, or take it every other day. Recheck your cholesterol levels in one month. If they have stabilized or continued to improve, you may no longer need the medication. If the levels begin to rise again, return to previous dosage. If you are currently on a cholesterol-lowering drug, you must consult your doctor before discontinuing the medication.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=712) | ||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||