|
Search Term: " Niacin "
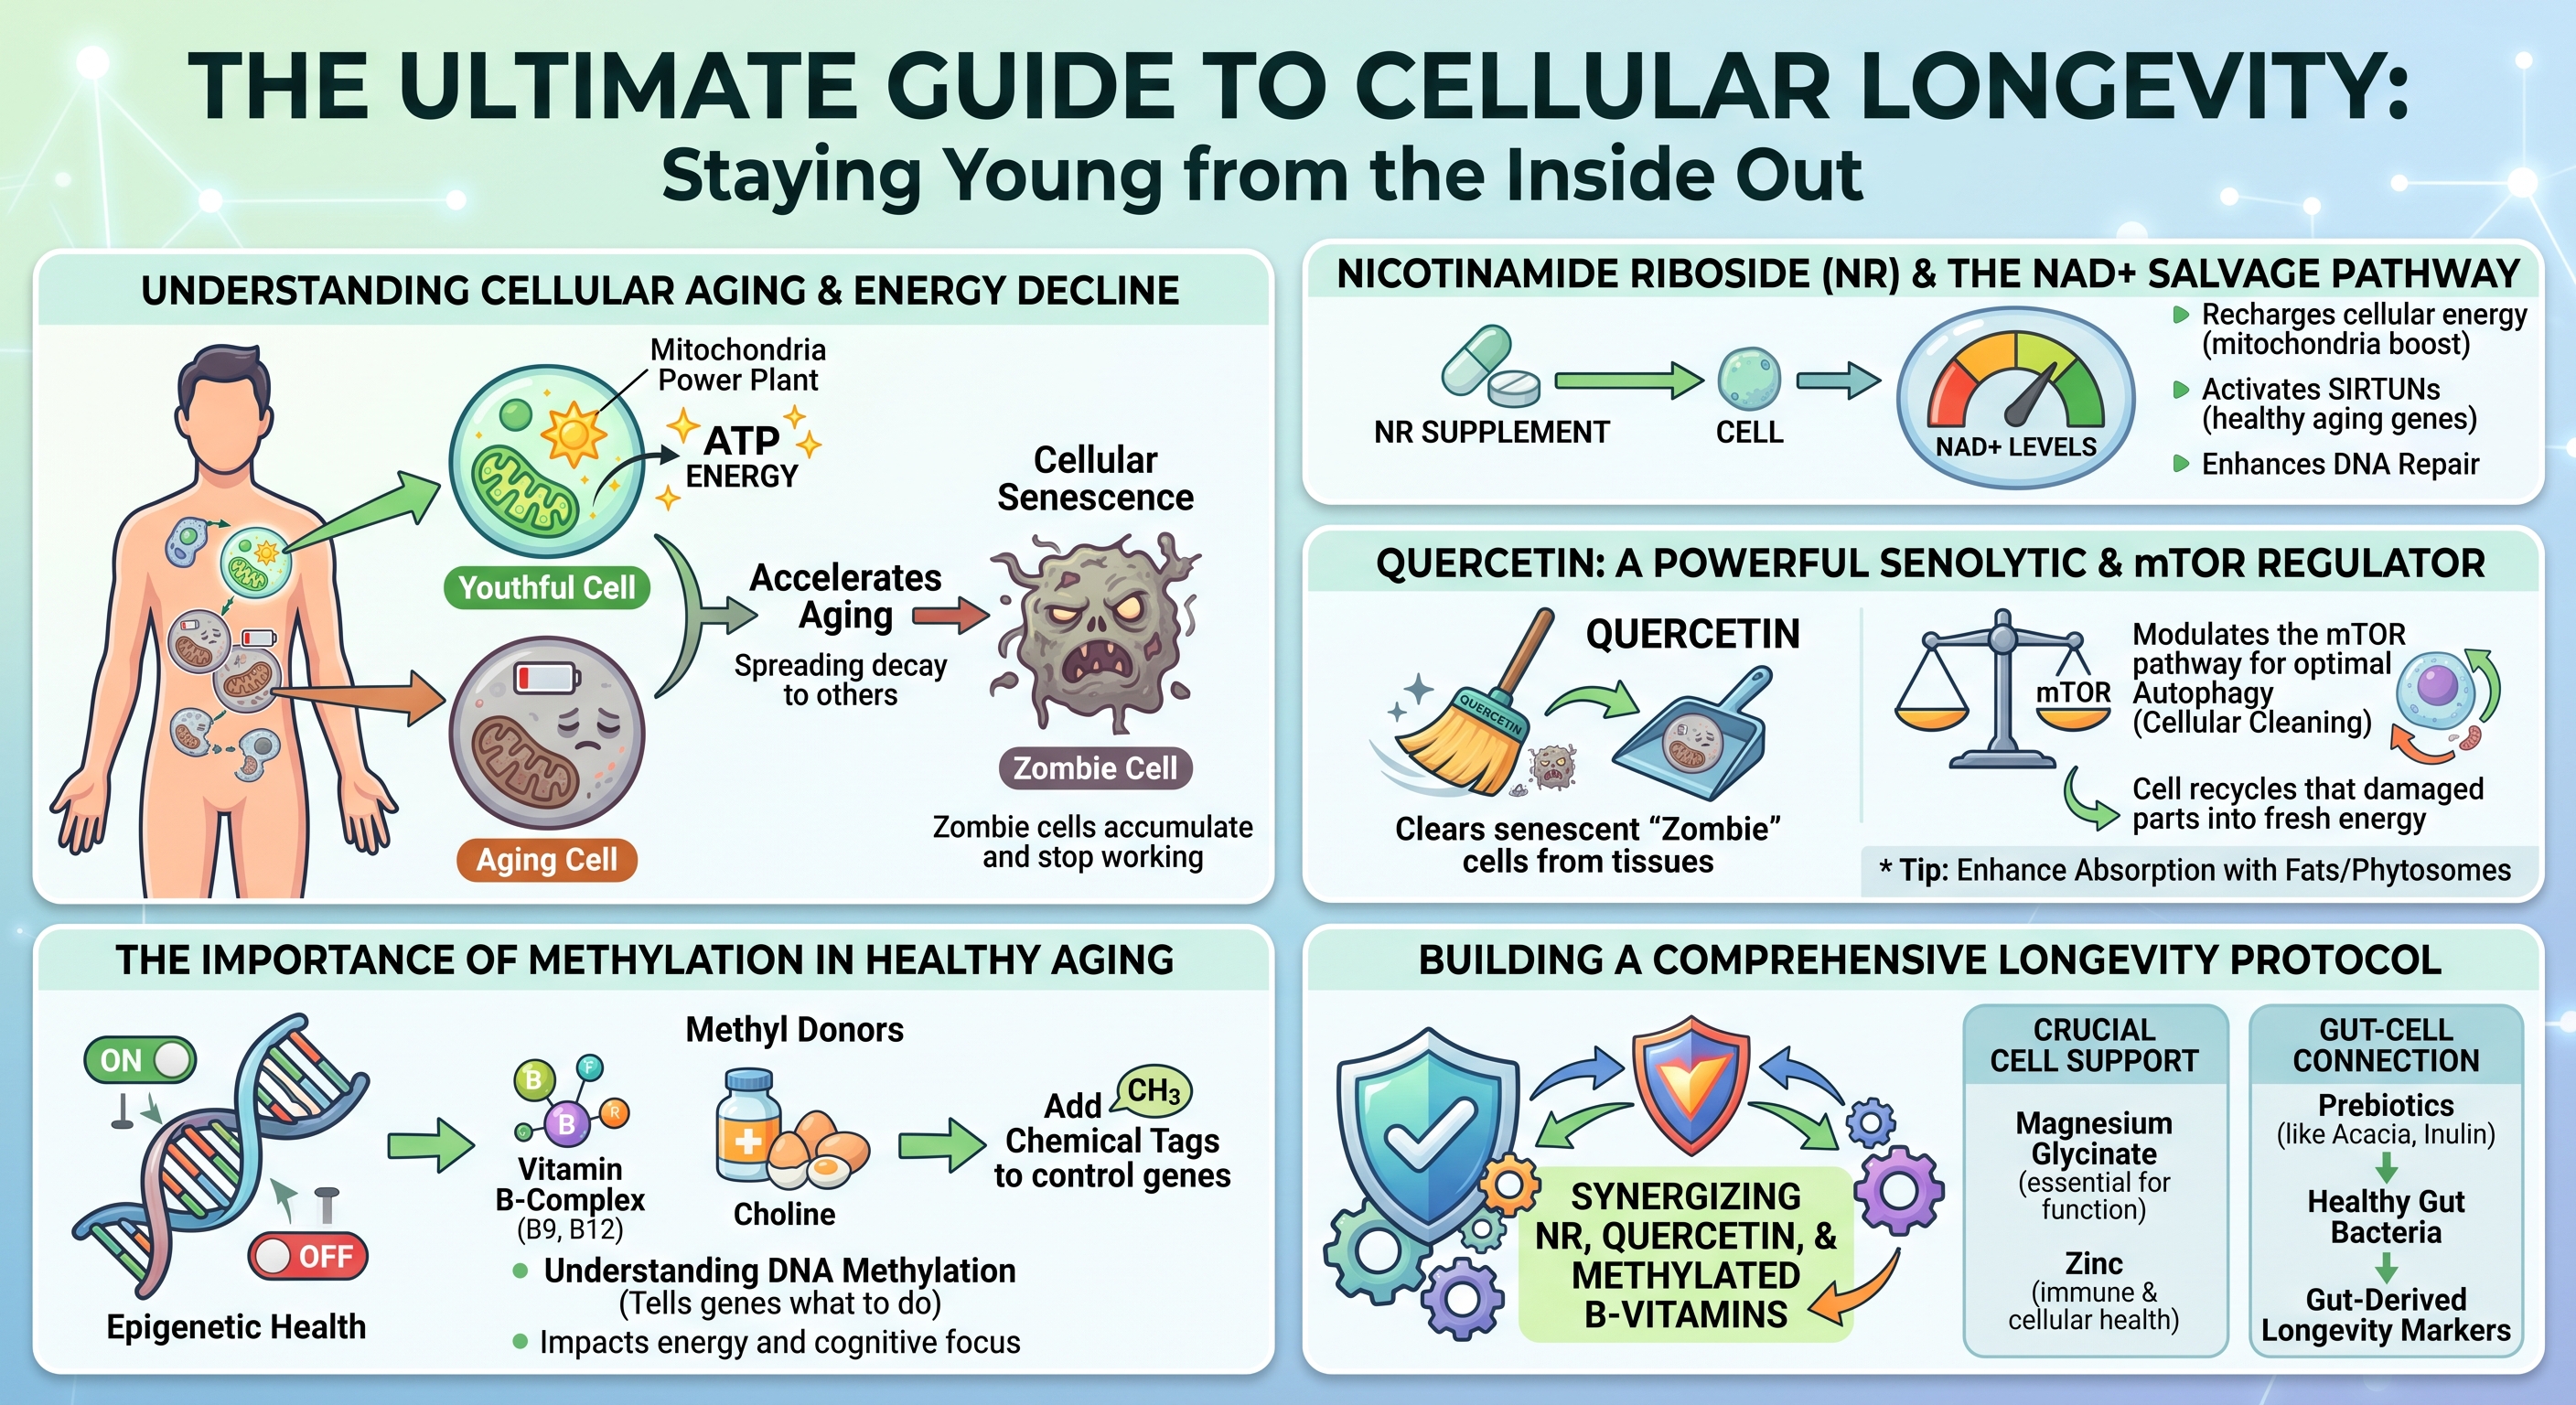
The Ultimate Guide to Cellular Longevity: NAD+, Methylation, and Senolytics   
Date:
September 10, 2026 10:57 AM
Introduction: Understanding Cellular Aging and Energy DeclineBiological aging represents a progressive decline in cellular maintenance, structural repair, and energy generation. Over decades, tissues experience an attrition of functional reserves, compromised stress resilience, and persistent low-grade systemic inflammation. At the cellular scale, biological degeneration is driven by a failure to generate bioenergetic fuel, repair genetic code, and clear metabolic waste.Cellular aging is characterized by interconnected biological disruptions known as the hallmarks of aging. These encompass genomic instability, epigenetic alterations, mitochondrial decay, loss of proteostasis, and cellular senescence. Rather than operating as isolated occurrences, these phenomena establish a self-reinforcing degenerative cycle: declining cellular power generation impairs enzymatic genetic repair, promoting the accumulation of damaged cells that enter irreversible growth arrest and poison surrounding healthy tissues. Mitigating cellular aging requires examining how microscopic bioenergetic pathways deteriorate and evaluating how targeted nutritional and biochemical interventions can restore cellular homeostasis. The Role of Mitochondria and ATP ProductionEvery biological function - from muscular contraction to continuous DNA replication - depends on adenosine triphosphate (ATP), the primary biochemical energy currency of living systems. Cells produce the vast majority of this energy within mitochondria through oxidative phosphorylation. Within these specialized organelles, metabolic intermediates derived from dietary carbohydrates and lipids donate high-energy electrons to the electron transport chain. The flow of these electrons across protein complexes establishes an electrochemical proton gradient across the inner mitochondrial membrane, driving ATP synthase to manufacture ATP.A youthful cell functions like an efficient municipal power grid, dynamically matching energetic demands with immediate ATP output. However, as biological aging progresses, mitochondrial efficiency declines. The electron transport chain becomes structurally leaky, inadvertently shedding electrons that react with ambient molecular oxygen to produce reactive oxygen species (ROS). While regulated levels of ROS participate in vital intracellular signaling, chronic excess induces widespread oxidative stress. Mitochondria are exceptionally vulnerable to this oxidative burden because they carry their own circular genetic material, known as mitochondrial DNA (mtDNA). Unlike nuclear DNA, mtDNA lacks the protective shielding of histone proteins and possesses rudimentary repair systems. As a result, mtDNA sustains cumulative oxidative damage, encoding increasingly defective electron transport chain proteins. This dynamic generates a bioenergetic deficit: degraded mitochondria synthesize progressively less ATP while emitting greater volumes of damaging free radicals. Deprived of optimal ATP reserves, cells lack the energy necessary to drive vital enzymatic repair cascades, accelerating structural degeneration and functional exhaustion. How Cellular Senescence Accelerates the Aging ProcessWhen healthy cells confront critical physiological damage - such as severe telomere attrition, persistent DNA double-strand breaks, or oxidative stress - they activate protective cell cycle arrest pathways governed primarily by the p53/p21^CIP1 and p16^INK4a/Rb molecular checkpoints. This defensive shutdown, termed cellular senescence, permanently prevents the replication of potentially premalignant or mutated cells.Senescent cells, colloquially known as "zombie cells," enter a state of permanent growth arrest while actively resisting programmed cell death (apoptosis). Over time, these cells accumulate within adipose depots, skeletal muscle, the vascular endothelium, and major organs, largely because immune surveillance and clearance pathways simultaneously lose functional efficiency. The systemic danger of senescent cells stems from their secretome. Rather than remaining biologically inert, senescent cells develop a hyperactive secretory state termed the Senescence-Associated Secretory Phenotype (SASP). The SASP is a destructive mixture of pro-inflammatory cytokines, chemokines, extracellular matrix-degrading matrix metalloproteinases (MMPs), and reactive oxygen species. Through this toxic secretome, even a small burden of senescent cells can impair whole-tissue architecture. SASP factors degrade surrounding structural proteins, induce insulin resistance in neighboring metabolic cells, and biochemically force adjacent healthy cells into secondary senescence. This persistent paracrine signaling fuels chronic, sterile, low-grade systemic inflammation, termed "inflammaging," which accelerates systemic tissue degeneration and elevates susceptibility to degenerative age-related pathologies. Nicotinamide Riboside (NR) and the NAD+ Salvage PathwayThe Biochemistry of NAD+ Depletion Over TimeNicotinamide adenine dinucleotide (NAD+) is an indispensable coenzyme present in every living cell. NAD+ fulfills a dual biological mandate: it serves as a central redox cofactor that shuttles electrons between cellular metabolic reactions, and it functions as an obligatory consumable substrate for regulatory enzymes that preserve cellular viability. In its redox capacity, NAD+ accepts electrons to form NADH during glycolysis, the tricarboxylic acid (TCA) cycle, and fatty acid beta-oxidation, subsequently donating those electrons to Complex I of the respiratory chain to power ATP synthesis.
The primary enzymatic driver of age-related NAD+ destruction is CD38, a membrane-bound glycohydrolase expressed on immune cells that is upregulated in response to chronic SASP exposure. Concurrently, lifelong genotoxic damage causes persistent activation of Poly(ADP-ribose) polymerase 1 (PARP-1), an enzyme that cleaves the glycosidic bonds of NAD+ to assemble branched poly(ADP-ribose) chains at DNA lesion sites. Because PARP-1 consumes NAD+ without directly recycling the molecule, chronic DNA damage depletes intracellular NAD+ pools, impairing bioenergetics and limiting sirtuin activity. How NR Efficiently Boosts Cellular NAD+ LevelsThe mammalian body maintains its NAD+ supply through three distinct biosynthetic routes: the de novo pathway from dietary L-tryptophan, the Preiss-Handler pathway from nicotinic acid (Niacin), and the NAD+ Salvage Pathway. The de novo pathway requires substantial energy expenditure, consuming roughly sixty milligrams of dietary tryptophan to yield a single milligram of NAD+. The Preiss-Handler pathway, while effective, can induce cutaneous prostaglandin-mediated flushing at therapeutic intakes. Consequently, the salvage pathway serves as the primary mechanism for maintaining intracellular NAD+ pools.The salvage pathway recycles the breakdown product nicotinamide (NAM), which is released whenever NAD+-consuming enzymes execute their functions. Under normal conditions, cells convert free nicotinamide into nicotinamide mononucleotide (NMN) via the rate-limiting enzyme nicotinamide phosphoribosyltransferase (NAMPT), after which NMN adenylyltransferases (NMNAT1–3) complete the conversion into NAD+. However, NAMPT expression declines with advancing age, chronic inflammation, and metabolic stress, limiting the recycling capacity of the cell. Nicotinamide Riboside (NR) is a naturally occurring pyridine nucleoside that bypasses this enzymatic bottleneck. Upon cellular entry via equilibrative nucleoside transporters, NR is directly phosphorylated into NMN by nicotinamide riboside kinases (NRK1 and NRK2) using a single molecule of ATP. Because the NRK pathway remains intact and robust across the lifespan, NR provides an efficient alternative entry point into the NAD+ salvage cascade. Clinical evaluations in humans confirm the safety, bioavailability, and pharmacokinetics of oral NR supplementation. Randomized, double-blind, placebo-controlled trials reveal that oral NR chloride produces dose-dependent increases in steady-state whole blood NAD+ concentrations. Dosing regimens of 100 mg, 300 mg, and 1,000 mg daily elevate blood NAD+ levels by approximately 22%, 51%, and up to 142%, respectively, within two weeks of administration, maintaining these elevations throughout continuous use. High-resolution metabolomic analyses also demonstrate parallel elevations in nicotinic acid adenine dinucleotide (NAAD), establishing it as a reliable biomarker of active intracellular NAD+ synthesis without hepatic or systemic toxicity. Sirtuin Activation and DNA Repair MechanismsReplenishing intracellular NAD+ supports functions beyond mitochondrial ATP generation. NAD+ functions as an obligatory cofactor for sirtuins (SIRT1 through SIRT7), a family of class III histone and non-histone protein deacetylases that regulate stress resilience, metabolic homeostasis, and cell survival. Sirtuins couple the removal of acetyl groups from target lysine residues to the stoichiometric cleavage of NAD+, producing nicotinamide and O-acetyl-ADP-ribose. In states of NAD+ deficiency, sirtuin enzymes remain inactive regardless of cellular demand.In the nucleus, SIRT1 coordinates defense against cellular decline. When activated by restored NAD+ levels, SIRT1 deacetylates peroxisome proliferator-activated receptor-gamma coactivator 1-alpha (PGC-1a), the master transcriptional coactivator of mitochondrial biogenesis. This deacetylation stimulates mitochondrial replication and assembly, expanding functional respiratory capacity. Concurrently, SIRT1 deacetylates the p65 subunit of nuclear factor-kappa B (NF-kB), suppressing the transcription of pro-inflammatory cytokines. In the mitochondria, SIRT3 utilizes NAD+ to deacetylate metabolic enzymes and superoxide dismutase 2 (SOD2), enhancing the organelle's capacity to neutralize reactive oxygen species. At the same time, cellular NAD+ levels directly regulate genomic integrity through PARP-1. When genotoxic stress or oxidative damage induces single- or double-strand DNA breaks, PARP-1 binds to the damaged termini using its zinc-finger domains. Bound PARP-1 hydrolyzes NAD+ to synthesize extensive, negatively charged poly(ADP-ribose) polymers on itself and adjacent histones. This modification relaxes chromatin architecture and establishes an electrostatic scaffold that recruits base excision repair and homologous recombination complexes. Recent discoveries demonstrate close crosstalk between sirtuins and PARP-1 during DNA repair. PARP-1 recruits SIRT1 to double-strand breaks, where SIRT1 deacetylates the chromatin-remodeling ATPase BRG1 to displace nucleosomes and facilitate homologous recombination. However, because PARP-1 and SIRT1 draw from the same intracellular NAD+ pool, severe NAD+ depletion forces a biological compromise: PARP-1 consumes the scarce remaining cofactor to address DNA damage, leaving sirtuins deactivated. Restoring NAD+ via NR prevents this deficit, enabling concurrent genomic repair and sirtuin-mediated metabolic defense. Quercetin: A Powerful Senolytic and mTOR RegulatorClearing Senescent "Zombie" Cells from TissuesThe accumulation of senescent cells has driven interest in senolytics: molecules that selectively eliminate senescent cells while sparing healthy, non-senescent populations. Senolytic agents exploit a specific vulnerability in senescent cells. Because senescent cells produce cytotoxic, pro-inflammatory SASP factors that would normally induce their own death, they become dependent on upregulated Senescent Cell Anti-Apoptotic Pathways (SCAPs) to survive. The SCAP network involves anti-apoptotic proteins (such as BCL-2 and BCL-xL), the PI3K/Akt kinase cascade, and cyclin-dependent kinase inhibitors.Quercetin is a polyphenolic flavonoid found in capers, red onions, apples, and the flower buds of Sophora japonica. Beyond its classical antioxidant properties, quercetin functions as a senolytic compound that exerts multi-target inhibitory effects across the SCAP network. By inhibiting the upstream PI3K/Akt survival axis and downregulating anti-apoptotic defenses, quercetin disrupts the signaling that protects senescent cells from intrinsic apoptosis. Deprived of these survival signals, senescent cells undergo programmed cell death. Preclinical studies demonstrate that senolytic protocols utilizing quercetin - often combined with the tyrosine kinase inhibitor dasatinib - reduce senescent cell burden across multiple tissues. This targeted clearance lowers circulating SASP factors, attenuates tissue fibrosis, restores endothelial reactivity, and improves functional health span. By removing senescent cells, quercetin mitigates the primary driver of chronic, low-grade inflammaging. Modulating the mTOR Pathway for Optimal AutophagyThe mechanistic Target of Rapamycin (mTOR) is an evolutionarily conserved serine/threonine protein kinase that coordinates cellular metabolism by balancing anabolic growth with catabolic recycling. Operating within two multiprotein complexes - mTORC1 and mTORC2 - the mTOR pathway integrates signals from amino acids, growth factors, and intracellular energy levels. In nutrient-rich environments, mTORC1 promotes protein synthesis, lipogenesis, and cellular growth, while suppressing catabolic breakdown. Conversely, nutrient scarcity downregulates mTORC1, activating autophagy.Autophagy is an intracellular degradation system that packages damaged organelles, misfolded protein aggregates, and biological debris into double-membraned autophagosomes for lysosomal degradation and recycling. A specialized branch of this pathway, mitophagy, selectively targets and clears damaged mitochondria. In modern metabolic conditions characterized by continuous caloric intake, mTORC1 can remain persistently active. This persistent signaling suppresses autophagy, causing damaged organelles and toxic aggregates to accumulate within tissues. Quercetin functions as a natural modulator of mTOR signaling. By inhibiting upstream PI3K/Akt signaling and activating intracellular energy sensors, quercetin attenuates overactive mTORC1, mimicking the metabolic effects of caloric restriction. This down-regulation relieves inhibition on the ULK1 autophagy initiation complex, stimulating both general autophagy and mitophagy. As autophagy proceeds, cells clear protein aggregates and eliminate damaged mitochondria, supporting cellular longevity and proteostasis. Enhancing Absorption: Phytosomes and Dietary FatsDespite the biological activities of quercetin identified in experimental models, its clinical translation has historically been limited by poor oral bioavailability. Raw quercetin aglycone is a crystalline, hydrophobic polyphenol with poor solubility in water and gastrointestinal fluids. When ingested in unformulated powder forms, quercetin molecules aggregate in the gut lumen, resisting dissolution and passive absorption. Consequently, the vast majority of an unformulated dose passes into the colon unabsorbed, where it undergoes microbial degradation without reaching meaningful systemic concentrations.To address these pharmacokinetic limitations, advanced delivery systems such as phytosomes were engineered. A phytosome is a 100% food-grade molecular complex where individual polyphenolic molecules are bound to dietary phospholipids, typically sunflower-derived phosphatidylcholine. Unlike a classical liposome - which encapsulates water-soluble compounds inside an aqueous core enclosed by a lipid bilayer - a phytosome forms an amphiphilic complex at the molecular level. The polar head of the phosphatidylcholine molecule forms hydrogen bonds with the hydroxyl groups of the quercetin molecule, while its lipophilic fatty acid tails extend outward. This structural arrangement shields the polar regions of the flavonoid, creating a lipid-compatible complex that integrates smoothly into the intestinal mucosa.
The Importance of Methylation in Healthy AgingVitamin B-Complex and Choline as Essential Methyl DonorsMethylation is an essential biochemical process occurring billions of times each second across all human tissues. It involves the transfer of a single-carbon unit - a methyl group consisting of one carbon atom bound to three hydrogen atoms - (CH3) - from a donor molecule to diverse recipients, including DNA, RNA, structural proteins, neurotransmitters, and membrane phospholipids. This transfer of one-carbon units is coordinated by the methionine-homocysteine cycle, which sustains genetic stability, detoxification pathways, and cellular repair.At the center of this pathway sits S-adenosylmethionine (SAM), the universal methyl donor in human biology. When a methyltransferase enzyme transfers a methyl group from SAM to an acceptor molecule, SAM is converted into S-adenosylhomocysteine (SAH). SAH functions as a potent competitive inhibitor of intracellular methyltransferases. To maintain functional methylation, SAH is rapidly hydrolyzed into homocysteine, a sulfur-containing amino acid that must be remethylated or cleared through transsulfuration. Homocysteine clearance proceeds through two distinct remethylation pathways. The primary route operates across most tissues via the enzyme methionine synthase, which requires vitamin B12 in its active methylcobalamin form. Methionine synthase transfers a methyl group from 5-methyltetrahydrofolate (5-MTHF, the active form of folate) to homocysteine, regenerating methionine. The ongoing production of 5-MTHF depends on the enzyme methylenetetrahydrofolate reductase (MTHFR), which utilizes riboflavin (vitamin B2) as a cofactor. Alternatively, excess homocysteine can be routed into the transsulfuration pathway by vitamin B6 (as pyridoxal-5'-phosphate) to synthesize cystathionine, cysteine, and ultimately the antioxidant glutathione. A secondary remethylation pathway, active predominantly in hepatic and renal tissues, bypasses folate entirely. In this route, dietary choline is oxidized to betaine (trimethylglycine or TMG). The enzyme betaine-homocysteine S-methyltransferase (BHMT) then transfers a methyl group from betaine directly to homocysteine, yielding methionine and dimethylglycine. When dietary intake of active B-vitamins or choline is insufficient, or when genetic variations like MTHFR polymorphisms reduce pathway flux, the methylation cycle slows. Homocysteine accumulates in circulation, promoting vascular and neurological inflammation, while SAM reserves decline, restricting cellular methylation capacity. Understanding DNA Methylation and Epigenetic HealthEvery somatic cell in an organism carries an identical genetic code. Cellular differentiation and tissue-specific functions are governed by the epigenome: a regulatory layer of chemical modifications that dictates gene expression without altering underlying DNA sequences. DNA methylation represents the primary and most stable epigenetic modification. In this process, DNA methyltransferase (DNMT) enzymes utilize methyl groups donated by SAM to add a methyl tag to cytosine bases adjacent to guanine residues, forming 5-methylcytosine within CpG dinucleotide sites.Under physiological conditions, DNA methylation maintains genomic stability and coordinates transcription. Methylation of promoter regions condenses chromatin, repressing transposable elements and silencing genes inappropriate for a given cell type. Conversely, hypomethylated promoters maintain an open chromatin state, allowing transcription factors to bind and initiate gene expression. During biological aging, this epigenetic landscape undergoes progressive dysregulation, a phenomenon termed "epigenetic drift". Aging cells experience global hypomethylation alongside focal hypermethylation of specific gene promoters. Global loss of methyl tags destabilizes the genome, activating retrotransposons and pro-inflammatory pathways. Simultaneously, hypermethylation at targeted promoter sites silences critical tumor suppressor genes and DNA repair complexes. This systematic change in DNA methylation patterns is consistent across populations, allowing researchers to develop molecular "epigenetic clocks". Algorithms such as the Horvath clock, PhenoAge, and GrimAge quantify biological age by profiling the methylation status of specific CpG sites across the genome. These clocks assess whether individuals are aging faster or slower than their chronological years. Ensuring a steady supply of methyl donors and preventing unnecessary SAM depletion supports DNMT activity, maintaining epigenetic patterns and genomic stability. How the Methylation Cycle Impacts Energy and Cognitive FocusBeyond long-term epigenetic regulation, the methylation cycle directly modulates immediate biochemical processes that govern daily energy, neurotransmission, and cognitive focus. Compromised methylation capacity frequently manifests as cognitive slowing, executive fatigue, and reduced physical stamina.A major consumer of methyl reserves is the endogenous synthesis of creatine. Approximately 40% of all SAM-derived methyl groups in the human body are utilized by guanidinoacetate N-methyltransferase (GAMT) in the liver to synthesize creatine. Creatine then translocates to the brain and skeletal muscle, where it is phosphorylated into phosphocreatine. Phosphocreatine functions as a rapid energy buffer, donating a high-energy phosphate group to regenerate ADP into ATP in milliseconds during demanding physical or cognitive tasks. When methyl donor availability falls, endogenous creatine synthesis drops, depleting phosphocreatine reserves and increasing susceptibility to neuromuscular and cognitive fatigue. Methylation is equally central to central nervous system architecture. SAM provides methyl groups to convert phosphatidylethanolamine into phosphatidylcholine, the predominant phospholipid comprising neuronal cell membranes and the myelin sheaths that insulate axons. Intact myelin preserves rapid action potential conduction throughout the nervous system. Furthermore, free choline derived from this pathway is the direct precursor to acetylcholine, the neurotransmitter required for attention, working memory, and learning. The methylation cycle also governs monoamine neurotransmitter metabolism. SAM is required for the synthesis of adrenaline (epinephrine) from noradrenaline, while catechol-O-methyltransferase (COMT) relies on SAM to degrade dopamine and norepinephrine within the prefrontal cortex. Sluggish methylation disrupts this balance, contributing to cognitive fatigue, mood variability, and impaired mental performance. Building a Comprehensive Longevity ProtocolSynergizing NR, Quercetin, and Methylated B-VitaminsLongevity supplementation often falters when single molecules are administered in isolation, ignoring interconnected metabolic pathways. Designing an effective cellular longevity protocol requires combining complementary mechanisms that reinforce one another while preventing secondary metabolic deficits. The combination of Nicotinamide Riboside, Quercetin Phytosome, and Methylated B-Vitamins illustrates this multi-target synergy.This synergy is grounded in the direct biochemical intersection between the NAD+ salvage pathway and the methylation cycle. When high-dose NR is supplemented to boost systemic NAD+, sirtuins and PARP enzymes consume the newly synthesized cofactor, generating substantial quantities of free nicotinamide (NAM). This intracellular nicotinamide faces two primary metabolic fates: it can be recycled back into NAD+ through the NAMPT-dependent salvage loop, or it can be cleared via methylation. When the influx of nicotinamide exceeds salvage recycling capacity, the excess is cleared to avoid feedback inhibition of sirtuin enzymes. To accomplish this, the enzyme nicotinamide N-methyltransferase (NNMT) transfers a methyl group from SAM directly onto nicotinamide, forming 1-methylnicotinamide (1-MNA/MNAM), which is subsequently excreted in urine. Prolonged, high-dose precursor administration without nutritional methyl support can elevate NNMT flux, depleting intracellular SAM reserves. As methyl groups are consumed clearing nicotinamide, the cellular SAM-to-SAH ratio falls, which can elevate circulating homocysteine and reduce methyl availability for DNA methylation and neurotransmitter synthesis. Co-administering a fully methylated B-complex alongside choline or betaine addresses this potential bottleneck. Providing active methyl donors (such as 5-MTHF, methylcobalamin, and betaine) maintains the one-carbon donor pool. Even during increased NNMT activity, SAM pools remain stable, protecting DNA methylation fidelity and maintaining homocysteine within safe parameters. Quercetin reinforces this protocol through complementary mechanisms. By clearing senescent cells and reducing SASP-mediated inflammation, quercetin downregulates CD38, the primary enzyme responsible for age-related NAD+ degradation. Suppressing CD38 prevents unnecessary breakdown of newly synthesized NAD+, enhancing the efficiency of NR supplementation. Furthermore, while NR provides the NAD+ necessary to activate SIRT1-driven mitochondrial biogenesis, quercetin concurrently modulates mTORC1 to stimulate autophagy. This coordinated action ensures that newly generated mitochondria operate in an environment cleared of proteotoxic cellular debris. The Crucial Role of Magnesium Glycinate and Zinc in Cellular FunctionLongevity protocols require essential mineral cofactors to function efficiently. Without adequate divalent minerals acting as enzymatic cofactors and structural stabilizers, metabolic longevity pathways cannot operate at full capacity. Among these, magnesium and zinc are required for cellular repair, genomic stability, and energy production.Magnesium serves as an obligatory cofactor in over 300 enzymatic reactions, primarily through its interaction with ATP. In biological systems, ATP exists predominantly as a chelate with a divalent magnesium ion, forming biologically active Mg2+ -ATP. Every enzymatic reaction that synthesizes, transfers, or consumes cellular energy - including the enzymes of the NAD+ salvage pathway (NRK and NMNAT) and DNA polymerases - strictly requires Mg2+ -ATP as its substrate. Magnesium deficiency impairs these phosphorylation reactions, reducing the cellular utilization of NAD+ precursors. Additionally, magnesium is an essential cofactor for the enzymes that activate dietary B-vitamins into their active forms. Supplying magnesium as magnesium glycinate provides high gastrointestinal bioavailability, minimal laxative effect, and yields glycine to support inhibitory neurotransmission and restful sleep. Zinc serves as a vital structural component for more than 3,000 human transcription factors and enzymatic proteins. Its most prominent structural role in longevity occurs within zinc-finger motifs. These are specialized protein conformations stabilized by a zinc ion coordinated to cysteine and histidine residues. The DNA damage sensor PARP-1 utilizes three zinc-finger domains to identify, track, and physically bind to single- and double-strand DNA breaks. Without adequate intracellular zinc, PARP-1 cannot properly assemble or dock onto damaged chromosomes, impairing DNA repair and increasing genomic instability. Zinc is also an obligatory structural component of copper/zinc superoxide dismutase (Cu/Zn-SOD or SOD1), the primary cytosolic antioxidant enzyme that dismutates superoxide radicals into hydrogen peroxide, protecting mitochondrial membranes and nuclear DNA from premature senescence. Integrating Prebiotics (like Acacia and Inulin) for Gut-Derived Longevity MarkersA comprehensive cellular longevity framework must extend beyond somatic tissues to encompass the gut microbiome. The intestinal microbiome functions as a central regulator of systemic inflammatory tone, immune development, and metabolic signaling. Age-associated dysbiosis - characterized by the loss of beneficial commensals and an overgrowth of pathobionts - frequently leads to breakdown of the intestinal barrier.The gut epithelium consists of a single-cell monolayer sealed by tight junction proteins, including zonula occludens-1 (ZO-1), occludin, and claudins. When this physical barrier is disrupted by poor dietary fiber intake or dysbiosis, gut permeability increases. This allows lipopolysaccharide (LPS), a component of the outer membrane of Gram-negative bacteria, to enter the portal and systemic circulation. The resulting "metabolic endotoxemia" activates Toll-like receptor 4 (TLR4) on immune cells, inducing NF-kB and systemic pro-inflammatory cytokine production. This persistent gut-derived inflammation exacerbates the SASP, accelerates tissue senescence, upregulates CD38, and drains systemic NAD+ reserves.
These short-chain fatty acids, particularly butyrate, exert direct protective effects on systemic longevity. Butyrate provides the primary metabolic fuel for colonic epithelial cells, supplying more than 70% of their baseline energy needs and supporting mitochondrial function within colonocytes. Furthermore, SCFAs upregulate the expression of epithelial tight junction proteins (ZO-1, occludin, and claudin-1), restoring intestinal barrier integrity and preventing the translocation of inflammatory LPS into systemic circulation. Systemically absorbed butyrate also functions as an endogenous histone deacetylase (HDAC) inhibitor, suppressing pro-inflammatory gene expression and supporting regulatory T cell (T_reg) development. Reducing metabolic endotoxemia dampens systemic inflammation, protecting vascular function and preventing premature NAD+ depletion. Conclusion: The Integrated Cellular Longevity MatrixCellular longevity is achieved not by addressing isolated biomarkers in isolation, but by systematically supporting interconnected biological pathways. As bioenergetic capacity declines, cellular senescence accelerates, epigenetic patterns degrade, and gut barrier integrity weakens. A comprehensive approach addresses these biological vulnerabilities simultaneously.
Quercetin Phytosome clears senescent cells and modulates mTORC1, stimulating autophagy while dampening the inflammatory SASP cascade that accelerates CD38-mediated NAD+ destruction. Methylated B-vitamins, active folate, and choline replenish SAM reserves, balancing the methyl requirements of NNMT-mediated nicotinamide clearance, preserving epigenetic DNA methylation, and maintaining neurotransmitter production. Magnesium glycinate and zinc provide the structural and catalytic foundation required for ATP utilization, B-vitamin activation, and PARP-1 zinc-finger DNA repair docking. Finally, prebiotic fibers generate short-chain fatty acids like butyrate, reinforcing the intestinal barrier and preventing metabolic endotoxemia from fueling systemic inflammation. By coordinating energy replenishment, cellular waste clearance, epigenetic maintenance, and the suppression of systemic inflammation, this unified approach directly addresses the underlying drivers of cellular aging to support long-term physiological vitality.
--
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=6650) NADH 10 mg And 20 mg Enhanced with Bioenergy RIBOSE 
Date:
December 10, 2009 04:23 PM
NADH 10 mg And 20 mg Enhanced with Bioenergy RIBOSE™
Based on a wealth of ongoing studies, we have a great understanding of the benefits of NADH. Not only is it an effective source of cellular energy, it is also one the body’s versatile electron donors—the molecule most frequently degraded during oxidation. Because of these characteristics NADH is, however, also very unstable with regard to light and oxygen, which leads to a very rapid loss of overall effectiveness. Additionally, poor lifestyle choices, such as the use of tobacco, excessive consumption of alcohol, drugs, and prescription medications, sleep deprivation, genetically-engineered foods, and a host of others can all inhibit the activity of NADH within the body. Hope is not lost, however. NOW® NADH contains a patented form of NADH from Panmol® - the first natural stabilized, stomach acidresistant form of this unique vitamin B3 supplement. Panmol® uses a patented process to naturally preserve its effectiveness. The end result is a highly stable, and bioavailable NADH which can easily withstand the harsh, acidic environment of the stomach and digestive tract; a breakthrough in the battle against many of todays’ most chronic conditions. NOW® NADH is available in both 10 and 20 mg potencies. Both varieties have been further enhanced with 200 mg of Bioenergy RIBOSE™ to support its cellular energy support properties.* Who Stands to Benefit from NADH With a proper supply of amino acids and/or B3 vitamins (Niacin) the human body is, in fact, capable of producing a limited reserve of NADH. Under chronic strain however, the body’s need for NADH increases. As we age, the body’s ability to manufacture NADH becomes increasingly limited. With this in mind, the following groups stand to benefit the most from incorporating NOW® NADH into their supplement regimen.
• Those who work in stressful, cognitively-demanding professions
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=2115) Vitamin B Complex
Date:
November 24, 2008 04:45 PM
The connection between B vitamin complex and stress is well known; although why a good B vitamin complex can reduce stress is less well known. Before discussing the reason why a Vitamin B formula can reduce stress, we shall first have a look at stress and what causes it. The term means different things to different people, and a stressful situation to one person might not be such to another. The biochemistry of stress is fairly complex, although involves the production and release of hormones into your bloodstream. When an event occurs that causes stress, the hypothalamus portion of your brain becomes involved. It releases cotocotropin releasing factor (CRF), a hormone that protects you from stress by raising your spirits. CRF sends signals to the pituitary gland causing the release of ACHT (Adrenocorticotropic hormone corticotropin) that causes cortisol to be released into the bloodstream by the adrenal glands. Cortisol speeds up the metabolism. Coincidentally, the cells of the brain stem and spinal cord send a message that stimulates the adrenal glands to secrete epinephrine that increases the heart rate, breathing and alertness, ready for fight or flight. Both of these mechanisms then lead back to the pituitary gland and your new stress level can repeat the process or stop it, should your stress be reduced. If this cycle continues over an extended period of time it can have serious repercussions on your mental and physical health. The B vitamins can help to regulate this biochemical function, and in doing so can reduce stress, and with it the associated anxiety and depression. In fact many of the symptoms of vitamin B deficiency are those that are also associated with stress: anxiety, nervousness, depression irritability and so on. There is no one specific form of Vitamin B that helps with stress, and there are eight in total. However, in saying that, the three members of the B vitamin complex that have most effect on stress are vitamins B 3, 6 and 12. Every one of the B vitamins is involved in cell metabolism. Because they are soluble in water, they are quickly leached from the body so have to be replaced on a regular basis. The various B vitamins are needed by your body for specific purposes, such as Vitamin B1 (thiamin) is essential for the correct function of your nerves, brain and muscles. Although others have their own particular areas of responsibility, they are generally lumped together, not only because they are all soluble in water, but also because they each have a profound effect on the metabolism of your body. Those mostly connected with the nervous system are Vitamins B3, B6 and B12. Vitamin B3 (Niacin) helps to maintain the proper health of your digestive system, skin and nerves, and B12 (cobalamin) is also needed for a healthy nervous system. Vitamin B6 (pyridoxine) along with vitamin B12 are the two principal members of the B complex that have an effect on stress, and a deficiency of these can make you more prone to this frequently debilitating condition. In fact many people that are suffering from a general Vitamin B deficiency have various forms of mental problems. Because Vitamin B12 is available only from animal sources, deficiencies are common in vegetarians, and even more common in vegans who are advised to take a Vitamin B12 supplement. However, in general you are best to take a Vitamin B complex as opposed to a supplement of any specific member of the B family. This is because a surplus of any one could lead to a depletion of others. It is thought that much of today's stress is caused by an inadequate diet, and a diet deficient in various forms of Vitamin B is believed to render the subject particularly prone to stress and anxiety. People that have been suffering undue levels of stress over a protracted period of time can be helped by a regular treatment of B vitamins. In taking such supplements, however, you should also be aware of the various possible effects on your body that the causes of your stress can have. These are frequently neither understood nor recognized when they occur. For example, if you are under stress due to a poor diet, or conversely, are eating a poor diet due to your high stress levels, you might be building up fatty deposits in your liver. Because of this your general health could be at serious risk in addition to your mental health. It is important, therefore, that you don't just restrict yourself to a B vitamin complex, but also take a supplement containing inositol and choline bitartrate. These can reduce the fatty deposit that a poor diet can cause to build up in your liver with consequent risk to life. Such deposits affect the ability of your liver to destroy the environmental toxins to which become exposed as part of your daily life, and which can be directly related to your ability to counter high stress levels. In general, however, if you are prone to stress and get nervous and worried about the slightest thing that doesn't go to plan, a B vitamin complex can help: vitamin B can reduce stress, although if your stress is sever you would be better advised consulting a physician than a health store. Stress is a serious condition, and not one that should be treated lightly. It is possible to treat some stress conditions by using a good B vitamin complex, although should the stress be serious then you should consult your physician. Frequently the stress is not diet related, but due to personal circumstances that cannot be cured by any form of supplement. However, there are few doubts that a course of Vitamin B supplements can help to overcome many of the metabolic causes of stress, and make up for any deficiency in these vitamins that leave your body almost as quickly as they enter it. Vitamin B can reduce stress, but only if your stress is due to a deficiency: and this is more common that most people are aware.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=1938) B Vitamin Complex
Date:
June 23, 2008 03:19 PM
The vitamin B supplement you take is a mixture of nutrients that, although they share the same vitamin letter, are in fact distinctly different chemical entities. The reason that they share the same reference letter of the alphabet is that they are all essential water soluble vitamins (Vitamin C being the only other), they frequently work in synergy with each other and they often come from common sources and have similar properties in the body. They were therefore at one time believed to be just the one chemical entity. They are essential in that they must form part of our diet because our bodies cannot manufacture these substances from others, and although most share common biochemical and health functions, there is no health function that requires all of them, and none of them can be totally replaced by another. The B-Vitamin complex that you take can consist of as many as eight different B vitamins, each of which is essential for a healthy body and at one time it was believed that this mixture was only one single vitamin. That is why they are collectively known as vitamin B and were subsequently allocated numbers: it was only later that the individual components were discovered. These eight are vitamin B-1 (thiamine), vitamin B-2 (riboflavin), vitamin B-3 (Niacin), vitamin B-5 (pantothenic acid), vitamin B-6 (pyridoxine), vitamin B-12 (cobalamins), biotin and folic acid (folate). They are found in yeast, liver, tuna, bananas and rice among other sources, and, as with all vitamins, without them life would not be possible. Not all vitamins are found in each of these food sources, and vitamin B-12, for example, is available in nutritional quantities only from animal sources. Knowing what they are is all very well, but what does your body do with the B vitamin supplement that you take? Before considering that, the reason that a regular supply is important is because of their water solubility. This is a useful property for a vitamin to possess, because it means that they can easily be transported by the body fluids to the tissues where they are needed. The downside, however, is that they are consequently also easily flushed from the body, and your body cannot store any of the B vitamins. You therefore must have a regular dietary source that can be augmented through supplementation. This is particularly desirable in alcoholics, those on diets to lose weight and vegans who are advised to take a regular vitamin B-12 supplement. A lack of vitamin B will make you feel tired and lack energy because they play a big part in your body’s metabolism of blood glucose into energy. They also help to maintain a healthy immune system, keep your nervous system in tip-top condition and maintain good healthy skin, hair and muscles. The B complex is also very important in maintaining healthy blood and liver, and each and every component of the mixture has a specific part to play, both on individually and by interaction with others in the B complex. Rather than examining what your body does with the supplement as a whole, let’s have a look at each component, and what your body does with that. Taking them one at a time, thiamine (B1) helps you to burn carbohydrates to generate energy. It is highly water soluble and must be taken daily. In the form of thiamine pyrophosphate it plays a key part in the metabolism of carbohydrates to energy, and also in the metabolism of certain amino acids. If you rely heavily on a high carbohydrate diet, you will need a good regular supplement of thiamine to be able to convert them to energy. Vitamin B2 (riboflavin) also plays a part in fat and carbohydrate metabolism and the formation of adenosine triphosphate (ATP), the molecule of energy. It plays a significant part in the health of your skin and a deficiency is associated with mouth ulcers, cracked lips, flaky skin and bloodshot watery eyes. It also activates vitamin B6 and folic acid, one of the cases where the B vitamins work together synergistically. Vitamin B3, or Niacin, is well known to women as a component of some shampoos, and helps to promote health hair. However, this vitamin also takes part in the process of energy creation within your body, and helps to maintain a good muscle tone within the digestive tract. It is also used as a supplement for the treatment of diseases related to high levels of LDL cholesterol and is useful for the treatment of atherosclerosis. Pantothenic acid is also found as a component of shampoos, so no prizes for guessing one of its functions. Vitamin B-5 plays a significant part in the energy-producing Krebs Cycle, or Citric Acid Cycle, that is used by every cell in your body to generate energy just where it is needed. It is also needed to synthesize acetylcholine, a neurotransmitter needed for good brain function and it helps to reduce stress. Pantothenic acid is also closely involved in the production of cholesterol in your liver: cholesterol is not all bad, and is needed by your body to produce some of the steroid hormones and also vitamin D. Amino acids are the small units that are used to biosynthesize proteins and ultimately the genes and DNA that determine who you are. The major factor involved in processing these amino acids is Vitamin B6 (pyridoxine), one of the lesser known of the vitamin B complex. It synthesizes and breaks up different amino acids to produce a variety of other compounds, such as the hormones serotonin, melatonin and dopamine. Deficiencies in these hormones can be very serious, Parkinson’s disease believed to be connected with a dopamine deficiency for example, and other disorders include kidney stones, anemia and many skin complaints. Although deficiency of vitamin B6 is rare, it can occur in alcoholics and those with chronic kidney problems. It is believed that many diets are deficient, however, and a good vitamin B supplement would ensure that this did not occur. Vitamin B-12 is one where deficiency can occur, particularly in alcoholics and vegans. It is available in sufficient quantities only from meat sources, and a supplement is indicated in anyone with a low meat intake in their diet. It is used by your body for the replication of DNA and to allow the normal activity of your body cells. It also helps to control homocysteine levels in conjunction with vitamin B6 and folic acid: homocysteine is a high-risk amino acid associated with atherosclerosis and cardiovascular disease that can lead to Alzheimer’s disease, heart attacks and strokes. The seventh, biotin (sometimes referred to as vitamin B7) also takes part in the metabolism of energy, but deficiencies have not been known, and the final known member of the B vitamin complex is folic acid. This is essential for cell growth and the synthesis of RNA and DNA in the body. RNA (Ribonucleic acid) is responsible for the synthesis of proteins in your body, and the well known Deoxy-ribonucleic acid (DNA) holds the genetic information of your body. Folic acid is therefore essential in the growing fetus, and any other cellular system that rapidly regenerates such as blood cells and the various cells of the immune system. Without folic acid your body would be more susceptible to bacterial and viral attack, and less able to protect you from foreign invaders into your body tissues. Although deficiency is not common, folic acid is present in fresh food only and degrades when stored at room temperature and when cooked. A supplement is therefore advisable during pregnancy to help to prevent neural tube defects. It is evident that the Vitamin B complex plays many parts in the chemistry of your body, and that a supplement can be of benefit in assuring that there are no deficiencies. A good B complex can be found at your local or internet health food store.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=1825) B Vitamin Supplements
Date:
May 07, 2008 03:18 PM
The fact that B vitamins have had to be coenzymated before they can be used by your body has been known for some time, but it is only over the past few years that they have been made commercially available in that form. Before we discuss the B vitamins in their coenzyme form it might be appropriate to discuss what coenzymes are and how they differ from ordinary enzymes. An enzyme is like an organic catalyst: it takes part in biochemical reactions by allowing such reactions to take place, but itself remaining unchanged. All enzymes are proteins formed in your body from amino acids and other protein material. A coenzyme, on the other hand, is somewhat like an enzyme for the enzymes, in that it is needed for the enzyme to do its job. Without a coenzyme, many enzymes could not promote the biochemical reaction it is responsible for. The B vitamins are all water soluble, which means that they are readily excreted and it is not impossible that if you take a B vitamin supplement, the whole lot will be immediately excreted in your urine if not used by your body. Whether they are or not it is a fact that your body can quickly become depleted of the B vitamin group, especially if you drink a lot. Alcoholics in particular are frequently vitamin B deficient. Although the liver can store unused vitamin B, they are only very small quantities and insufficient to prevent a deficiency. A deficiency in the B vitamins can cause a wide range of unpleasant conditions that are rapidly remedied with supplements. Pellagra is due largely to a deficiency in Vitamin B3, and causes hair loss, horrible skin lesions and many other side effects that you don’t want to know about. Vitamin B12 deficiency can cause loss of memory, and is common in alcoholics and some vegetarians (vitamin B12 is animal derived). Other symptoms of a general B vitamin deficiency include exhaustion, heart palpitations, fibrillation, anxiety, restlessness, attention deficit disorder and many, many more. It is not pleasant so you make sure that take enough vitamin B in your diet: dietary sources are far superior to pills although supplements will help you get over the symptoms of the deficiency until your diet takes over. Supplementation is also a good way to maintain a regular supply of vitamin B complex irrespective of your diet. The effects of a deficiency are so bad that a regular supplement is well worth taking. However, back to coenzymes and why they are needed for the metabolism of B vitamins in your body. Most B vitamins are, in fact, coenzymes themselves. Keep in mind that the definition of a vitamin is an organic substance that is essential for the normal health of your body. If you lack even one vitamin, your health with suffer and eventually you will be likely to die. That describes all of the B vitamins perfectly, and they also just happen to be coenzymes. This is not coincidence, of course, and their biochemistry must have been recognized before the concept of coenzymes was formulated. The B vitamins proper consist of eight distinct proteins: B1 (thiamine), B2 (riboflavin), B3 (Niacin), B6 (pyridoxine), B9 (folic acid), B12 (cyanocobalamin), and biotin and pantothenic acid. They are all essential components in human and animal metabolism, and most are also coenzymes. Every cell in your body depends on B vitamins for its existence, which is why pregnant women should include a good supply of them in their diet, especially folic acid (B9). They are essential for the cellular development of the fetus. Folic acid is necessary for the synthesis of nucleic acids that allow cell growth and the production of red blood cells. However, not one can be placed in importance above any other since they are all essential. With respect to the coenzyme factor, the vitamin B coenzymes are responsible for many of the biochemical reactions upon which life depends. Coenzyme B-12 for example is essential for two types of reaction that it catalyzes, one being a hydrogen atom exchange with alcohol and amine functional groups, the other being connected with methyl group transfer between molecules. In humans, the first of these is responsible for an essential step that results in energy being metabolized from fats and proteins in the mitochondria and the second for DNA production in cells that is indirectly responsible for growth. Each of these is why a vitamin B-12 deficiency leads to excessive fatigue and also a lack of fetal growth (although folic acid can make up for the latter deficiency). Thiamine (Vitamin B1) is a coenzyme for the metabolism of carbohydrates to energy. In the body it is present in the form of thiamine diphosphate, a coenzyme that assists in the decarboxylation of pyruvate as part of the citric acid cycle, otherwise known as the Krebs Cycle, that takes place in the mitochondria and is responsible for the generation of energy through aerobic respiration. Another coenzyme that is involved in the Krebs Cycle is formed in the body from Vitamin B3, or Niacin. This coenzyme, nicotinamine adenine dinucleotide, has a redox potential and can store energy for use later on. Vitamin B5 can be converted in the body to Coenzyme A that not only breaks proteins down into individual amino acids, but also takes part in the first part of the Krebs Cycle. There is a common pattern emerging here where the B vitamins have an important part to play in the generation of energy from fats and carbohydrates. Similarly, Vitamin B6 is present in the body as the coenzyme Pyridoxal 5'-phosphate that helps to break down the body’s emergency energy store, glycogen, into energy when needed. In these ways, and more, the coenzymes created in the body from the B vitamins help many of the reactions of life to take place, and without these coenzymes life could not exist. Hence the importance of the B vitamins themselves, and any deficiency could be disastrous to the metabolic processes that generate energy and keep you alive. It is not just the energy needed for exercise and normal human activity that will be compromised, but also that which keeps the heart beating and your diaphragm moving to allow you to breath.
Without a doubt, a Vitamin B supplement is one of the most valuable of all the vitamin supplements, and they are available in many forms. You might also find some of the B vitamins in their coenzyme form, though some of them may be unstable. However, whatever form they are taken in, Vitamin B complex should be one of the first on your vitamin supplement shopping list.
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=1784) Cholestrex - Lower Cholesterol with Source Naturals Supplements 
Date:
June 01, 2005 10:41 AM
Our lives depend on an uninterrupted flow of blood throughout the 60,000 miles of arteries, veins, and capillaries that bring vital nourishment to our cells. Our bodies have complex chemical strategies to maintain and repair blood vessel walls. Cholesterol is an important part of the process. However, too much cholesterol in the bloodstream can have serious consequences for our well-being. By understanding how nutrition affects blood cholesterol, we can gain valuable control of our health. Source Naturals CHOLESTREX has been formulated to provide the nutritional support that we need to maintain healthy cholesterol levels. SINCE DOCTORS FIRST DISCOVERED that cholesterol was the primary ingredient in the sticky deposits that clogged their patients’ arteries, scientists have gained a thorough understanding of cholesterol’s role in our health. Essential to human and animal life, cholesterol is part of every cell in the body. Because cholesterol is so important, the liver synthesizes from 1 to 2 grams of it each day. In addition, we get about another 500 mg from the foods we eat. Problems occur when too much cholesterol gets into the bloodstream. Today, it’s estimated that over 50 million adults in the United States have cholesterol levels that are too high. The body’s processes to manage excess cholesterol depend upon a lifestyle that includes exercise, stress reduction and proper nutrition. Source Naturals Cholestrex is designed to deliver a comprehensive combination of nutrients known to support a healthy blood vessel system – and keep the life stream flowing.
The nutrients in CHOLESTREX are known to support a healthy blood vessel systemCholesterol: What It Is Cholesterol is a solid waxy substance, technically classed as a “sterol.” Cholesterol enables our cell membranes to maintain their integrity. It is the basic raw material from which the body makes steroid hormones, which include the sex hormones. Cholesterol is the primary component of bile salts that the liver creates to help us assimilate fats, fat-soluble vitamins and essential fatty acids. The liver also uses bile to rid itself of stored toxins. Our skin contains large amounts of cholesterol, making it resistant to the absorption of water-soluble toxins. Even the brain is 7% cholesterol (dry weight).
Blood vessel walls cover a surface area of half an acre and are under constant pressureCholesterol in the Blood Because it’s not water-soluble, cholesterol must be attached to a carrier molecule in order to be transported in the bloodstream. The liver manufactures two types of carrier molecules for cholesterol, LDL and HDL. LDL (low density lipoprotein) molecules carry cholesterol from the liver out to cells of the body. One of its functions is to repair damaged cells, including those of the artery walls. LDL is primarily made up of saturated fats, (meat fats, butter, etc.). HDL (high density lipoprotein) molecules transport cholesterol and fatty acids from body tissues back to the liver for disposal. HDL helps remove excess fat and cholesterol from the bloodstream. HDL is composed of liquid fats (most vegetable oils). It’s crucial to have a proper balance between LDL and HDL cholesterol. High LDL – a sign that the body has too much fat – is a threat to the health of blood vessels, because excess LDL cholesterol may accumulate in damaged areas of vessel walls. These “fatty streaks” are the beginning stage of artery blockage.
The oxidation of LDL cholestrol is at the heart of the problemCholesterol and Artery Damage The walls of the blood vessels cover a surface area of half an acre and are under constant pressure. Of all the blood vessels in the body, the coronary arteries are under the greatest stress. Named for the Latin word for crown (corona), they sit directly on the heart muscle and must continually expand and contract with every heartbeat. That’s 100,000 times each day. This constant squeezing can cause small lesions in the artery wall. This triggers a repair process where LDL cholesterol comes in to patch up the damage. Recent research has found that the crux of the problem is the oxidation of LDL cholesterol. Rich in fatty acids, the LDL molecule becomes permanently altered when oxidized by free radicals (overreactive molecules that steal electrons from other molecules). These rancid, oxidized LDL molecules are no longer recognized by the body, so they’re attacked by immune system cells. These immune cells become bloated with the oxidized lipids, accumulate in artery lesions and create plaque in blood vessels. Why is LDL cholesterol being oxidized? First of all, there’s too much of it in the blood, while not enough HDL. Secondly, the blood doesn’t have enough antioxidants to neutralize free radicals. The ingredients in Source Naturals Cholestrex address these specific problems in several ways. Cholestrex also provides nutrients that protect and strengthen blood vessel walls.
In the typical American diet, 95% of the cholesterol meant for removal is reabsorbedCholestrex Has It All Vitamin C helps maintain the health of artery walls because it’s the key building block for collagen and elastin, the primary constituents of blood vessels. Copper is required by the enzyme that weaves together the fibers of collagen and elastin into the matrix that makes vessel walls both tough and flexible. As an antioxidant, vitamin C scavenges free radicals in the blood plasma and also regenerates vitamin E within the LDL molecule. Vitamin E has a critical role as the primary protector of LDL, preventing its oxidation. One molecule of vitamin E can protect 200 molecules of polyunsaturated fatty acids from free radical damage. GTF Chromium is involved in insulin activity and the normalization of blood sugar. Excess simple sugars are converted to triglycerides, the blood fats which can accumulate in artery walls. Lecithin is a component of HDL that emulsifies excess blood fat so it can be more readily transported in the bloodstream to the liver, where it’s metabolized. Vitamin B3 (Niacin) assists in the metabolism of fats, and puts an electric charge on red blood cells so they repel each other, which prevents blood clumping. The amino acid, L-Arginine, works to lower serum cholesterol and triglycerides by inhibiting fat absorption.
Beta sitosterol neutralizes incoming dietary cholesterolThe Body’s Cholesterol Removal System HDL molecules carry cholesterol from tissues throughout the body back to the liver, where it is incorporated into bile salts. These bile salts are sent to the intestines, where they combine with fiber for excretion. One problem with the typical American low fiber diet is that 95% of the bile-bound cholesterol is reabsorbed. Since this is the body’s primary pathway for ridding itself of excess cholesterol, another strategy incorporated into Cholestrex is to maximize the production of bile salts and minimize their reabsorption by increasing levels of fiber. Fiber is a key element of Cholestrex. Its four types of soluble fiber bind with bile salts that are laden with cholesterol to ensure their excretion from the body. Oat Bran & Fiber, Grapefruit Pectin, Psyllium Seed Husks and Alfalfa Seeds also absorb cholesterol from our food, thereby lowering total blood cholesterol. Alfalfa seeds are considered a blood purifier. Beta sitosterol, a plant equivalent of cholesterol, binds to sites in the intestines that would otherwise absorb cholesterol. Cholestrex provides a daily total of 300 mg of beta sitosterol which may, by itself, neutralize 200 to 300 mg of incoming dietary cholesterol by preventing its absorption. Vitamin C, among its many other vital roles, is the key factor in activating an enzyme that will increase the liver’s conversion of cholesterol into bile salts. CHOLESTREX uses bioactive mineral ascorbate forms of vitamin C that will not irritate the digestive system. Working in conjunction with the fiber in CHOLESTREX, Calcium increases HDL, while lowering total serum cholesterol. Cholestrex–Intelligent Nutritional Support Our generation is fortunate to witness the remarkable progress made by modern science in understanding the body’s complex biochemical processes. As we realize the vital connection between nutrition and cholesterol levels, we are empowered to improve our health and vitality beyond previous standards of wellness. Source Naturals CHOLESTREX. For you and the ones you love.
Reference:
(https://vitanetonline.com:443/forums/Index.cfm?CFApp=1&Message_ID=132) | ||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||||


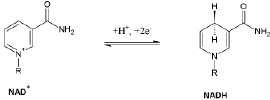 NADH is the biologically-active form of vitamin B-3 (Niacin), and is involved in a wide range of functions throughout the body. An easier way to understand it, is to think of NADH as a biological spark plug that makes it possible for us to become and remain energetic, active, and functioning at our best. Remove the “spark” and some of the most basic human functions will inevitably suffer. This is not speculation. It is the result of decades of scientific investigation that has examined the link between nutrition and chronic conditions; notably those related to cellular life cycles and apoptosis, excessive fatigue, enzyme decline, free radical expansion, cognitive disparity, intracellular balance, normalized aging, and many more important aspects of human health.*